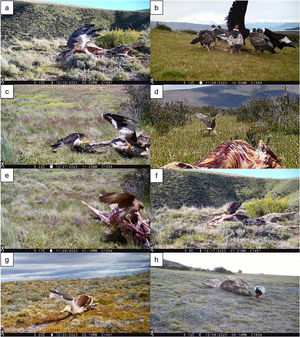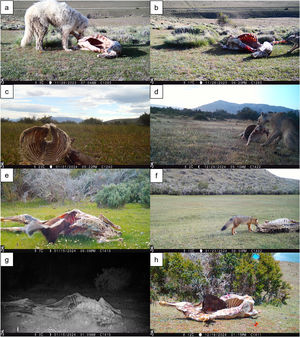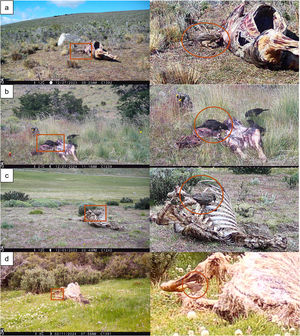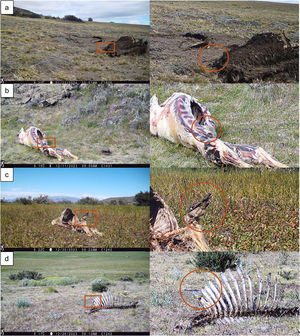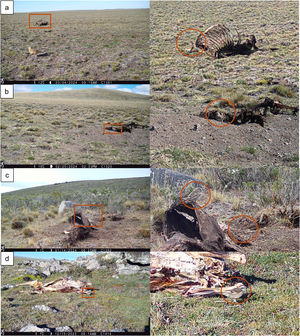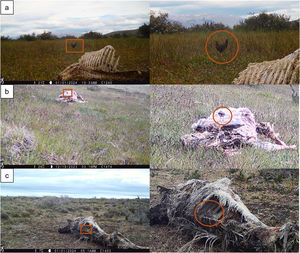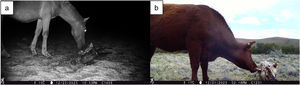


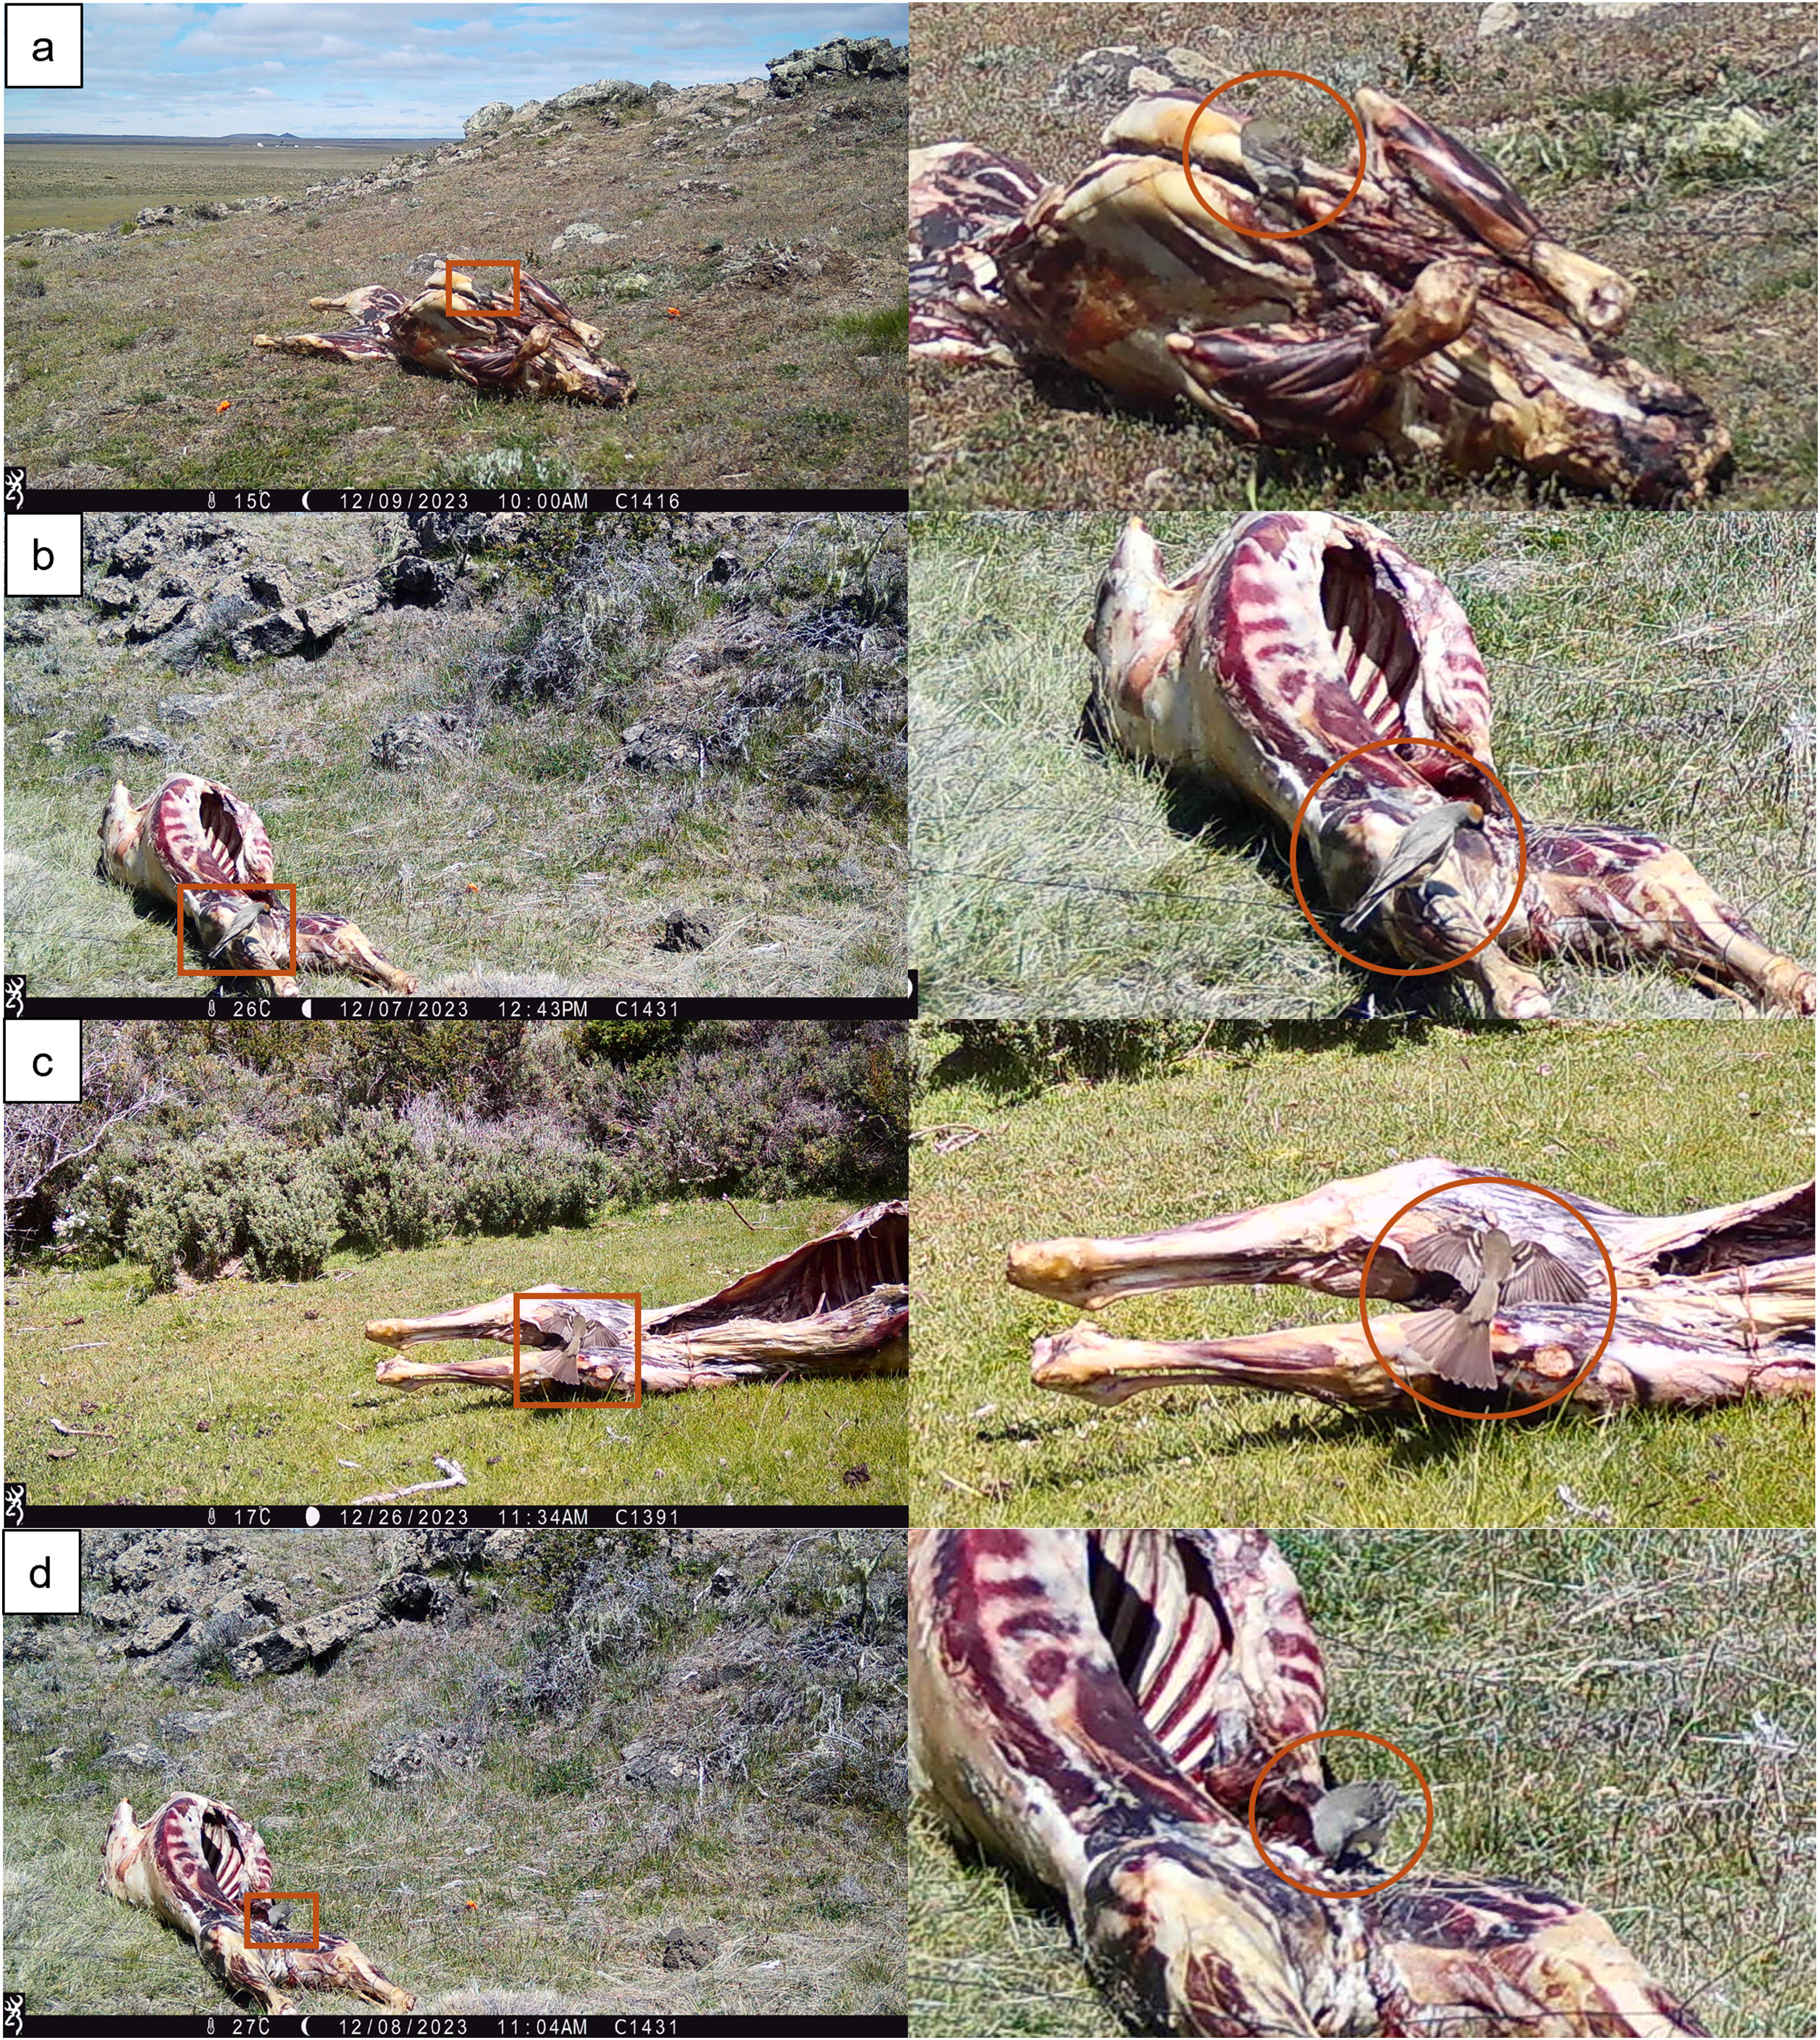
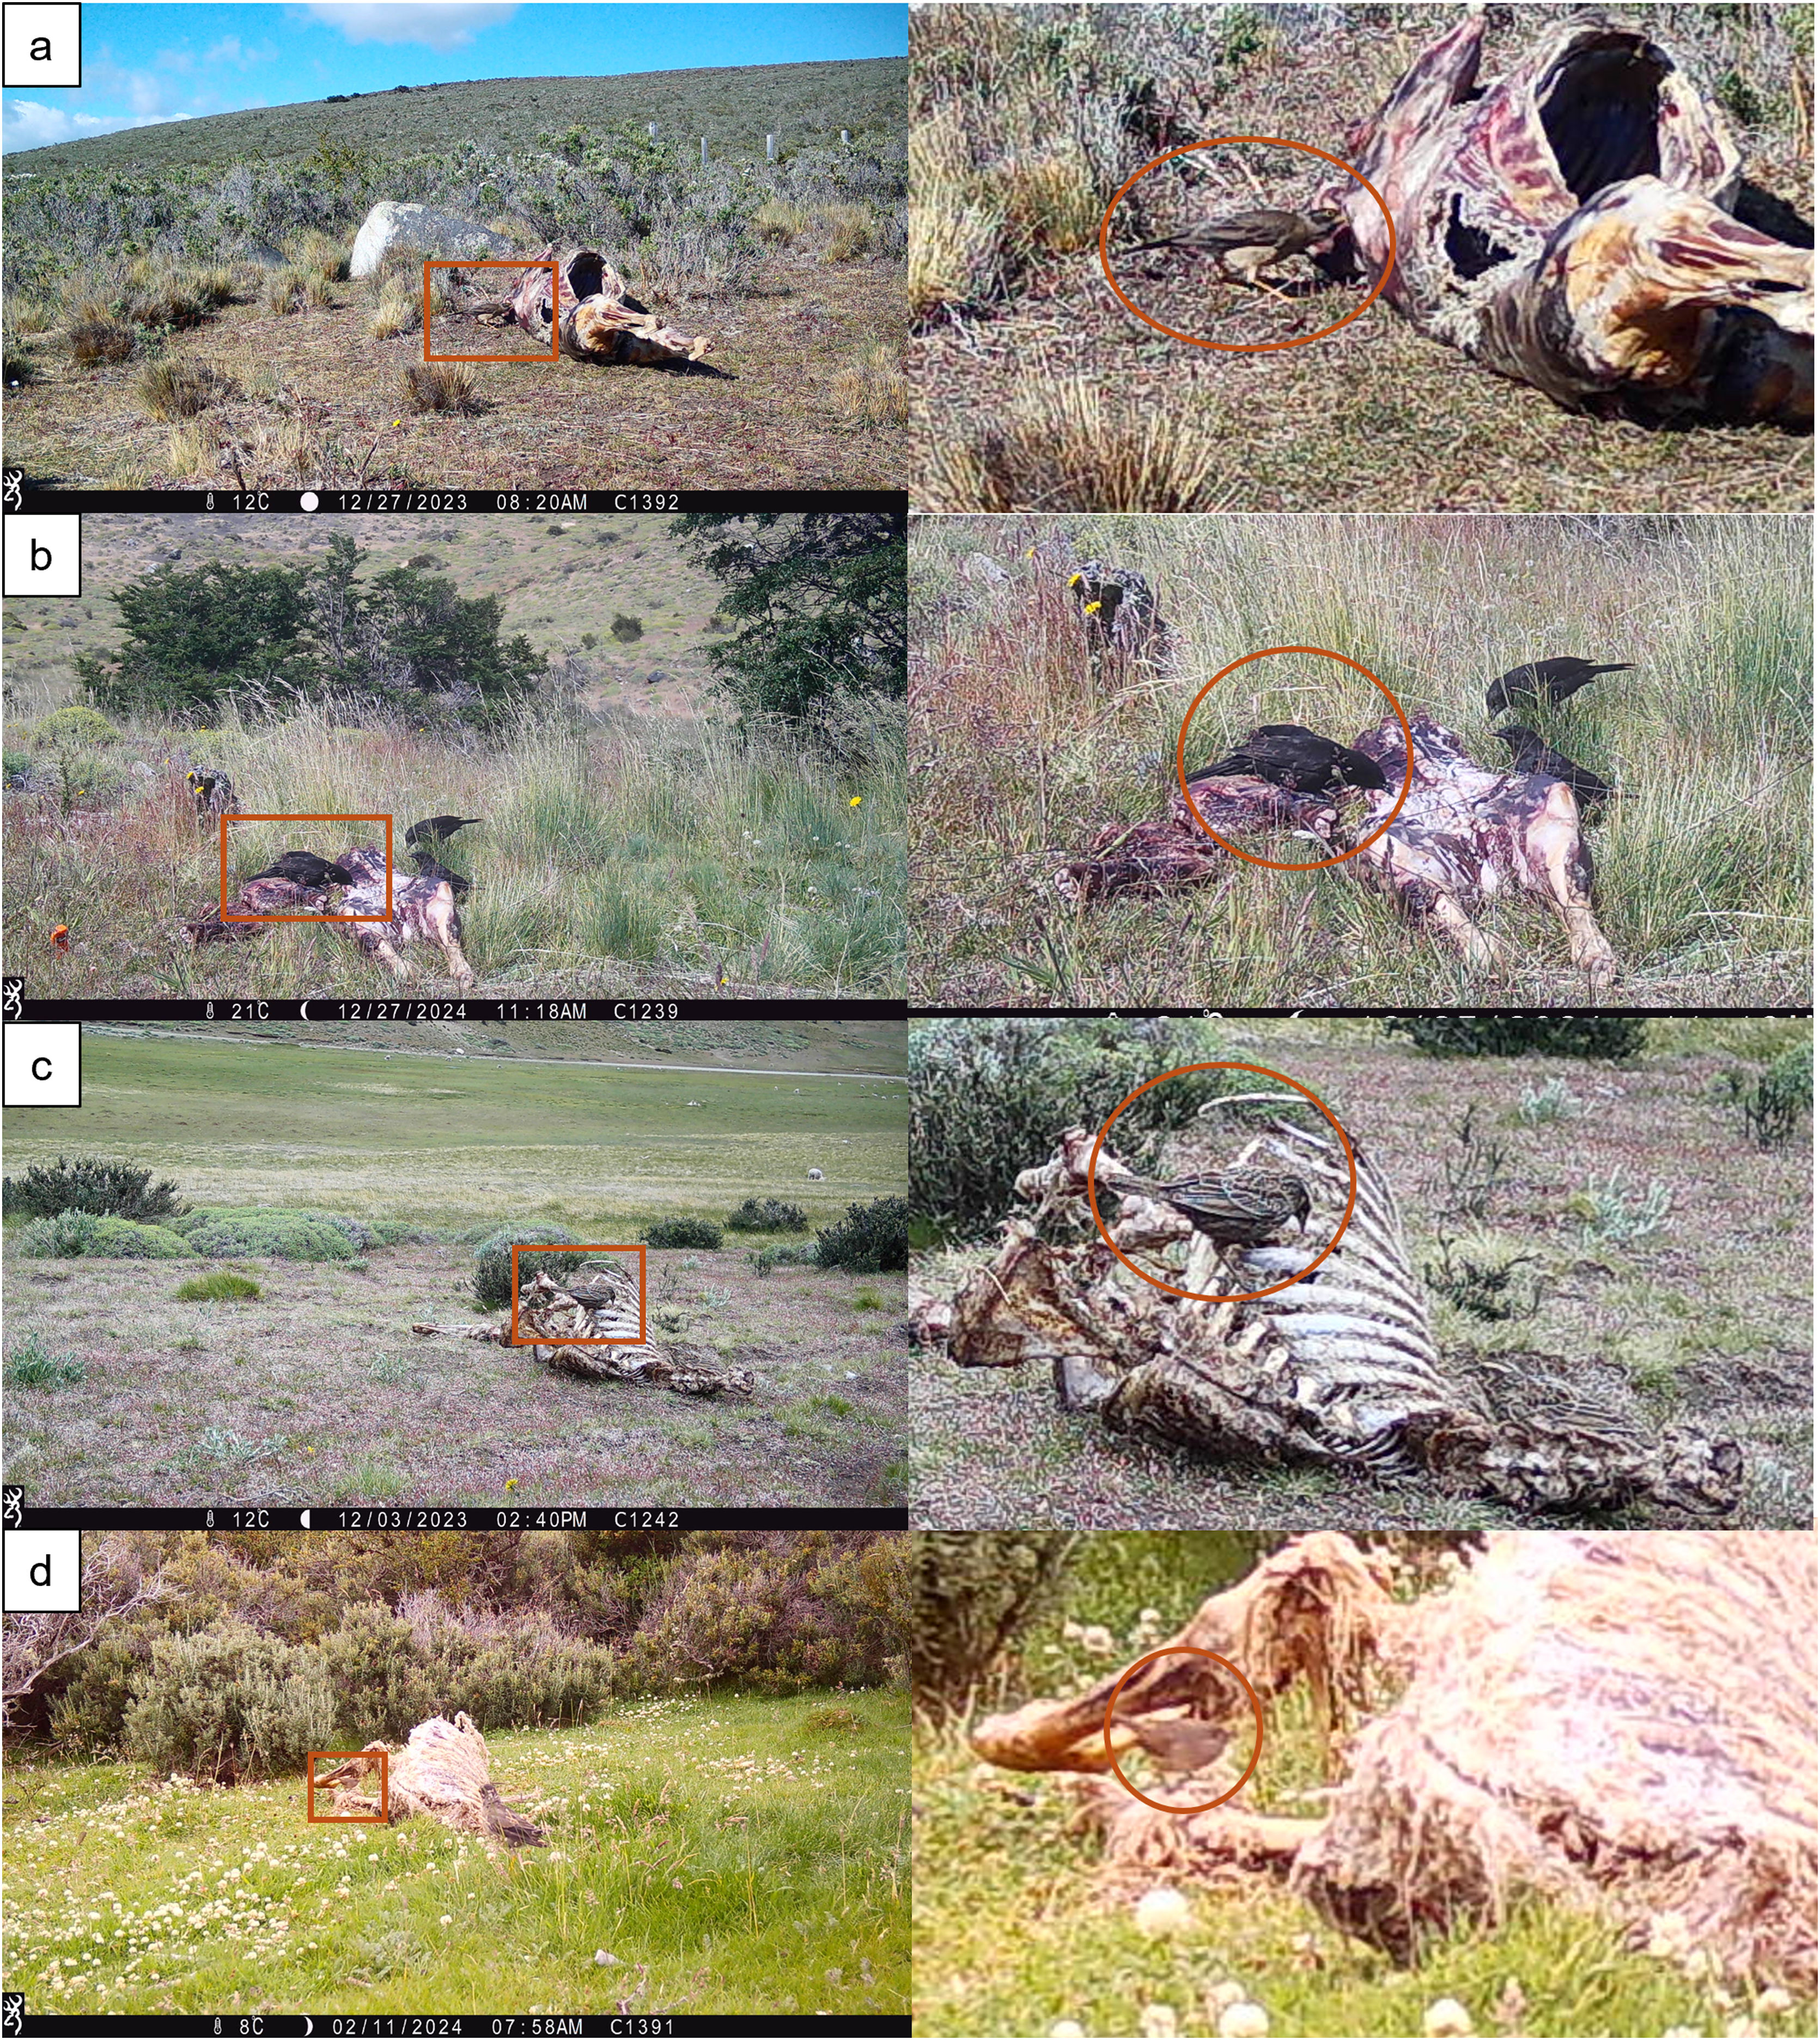
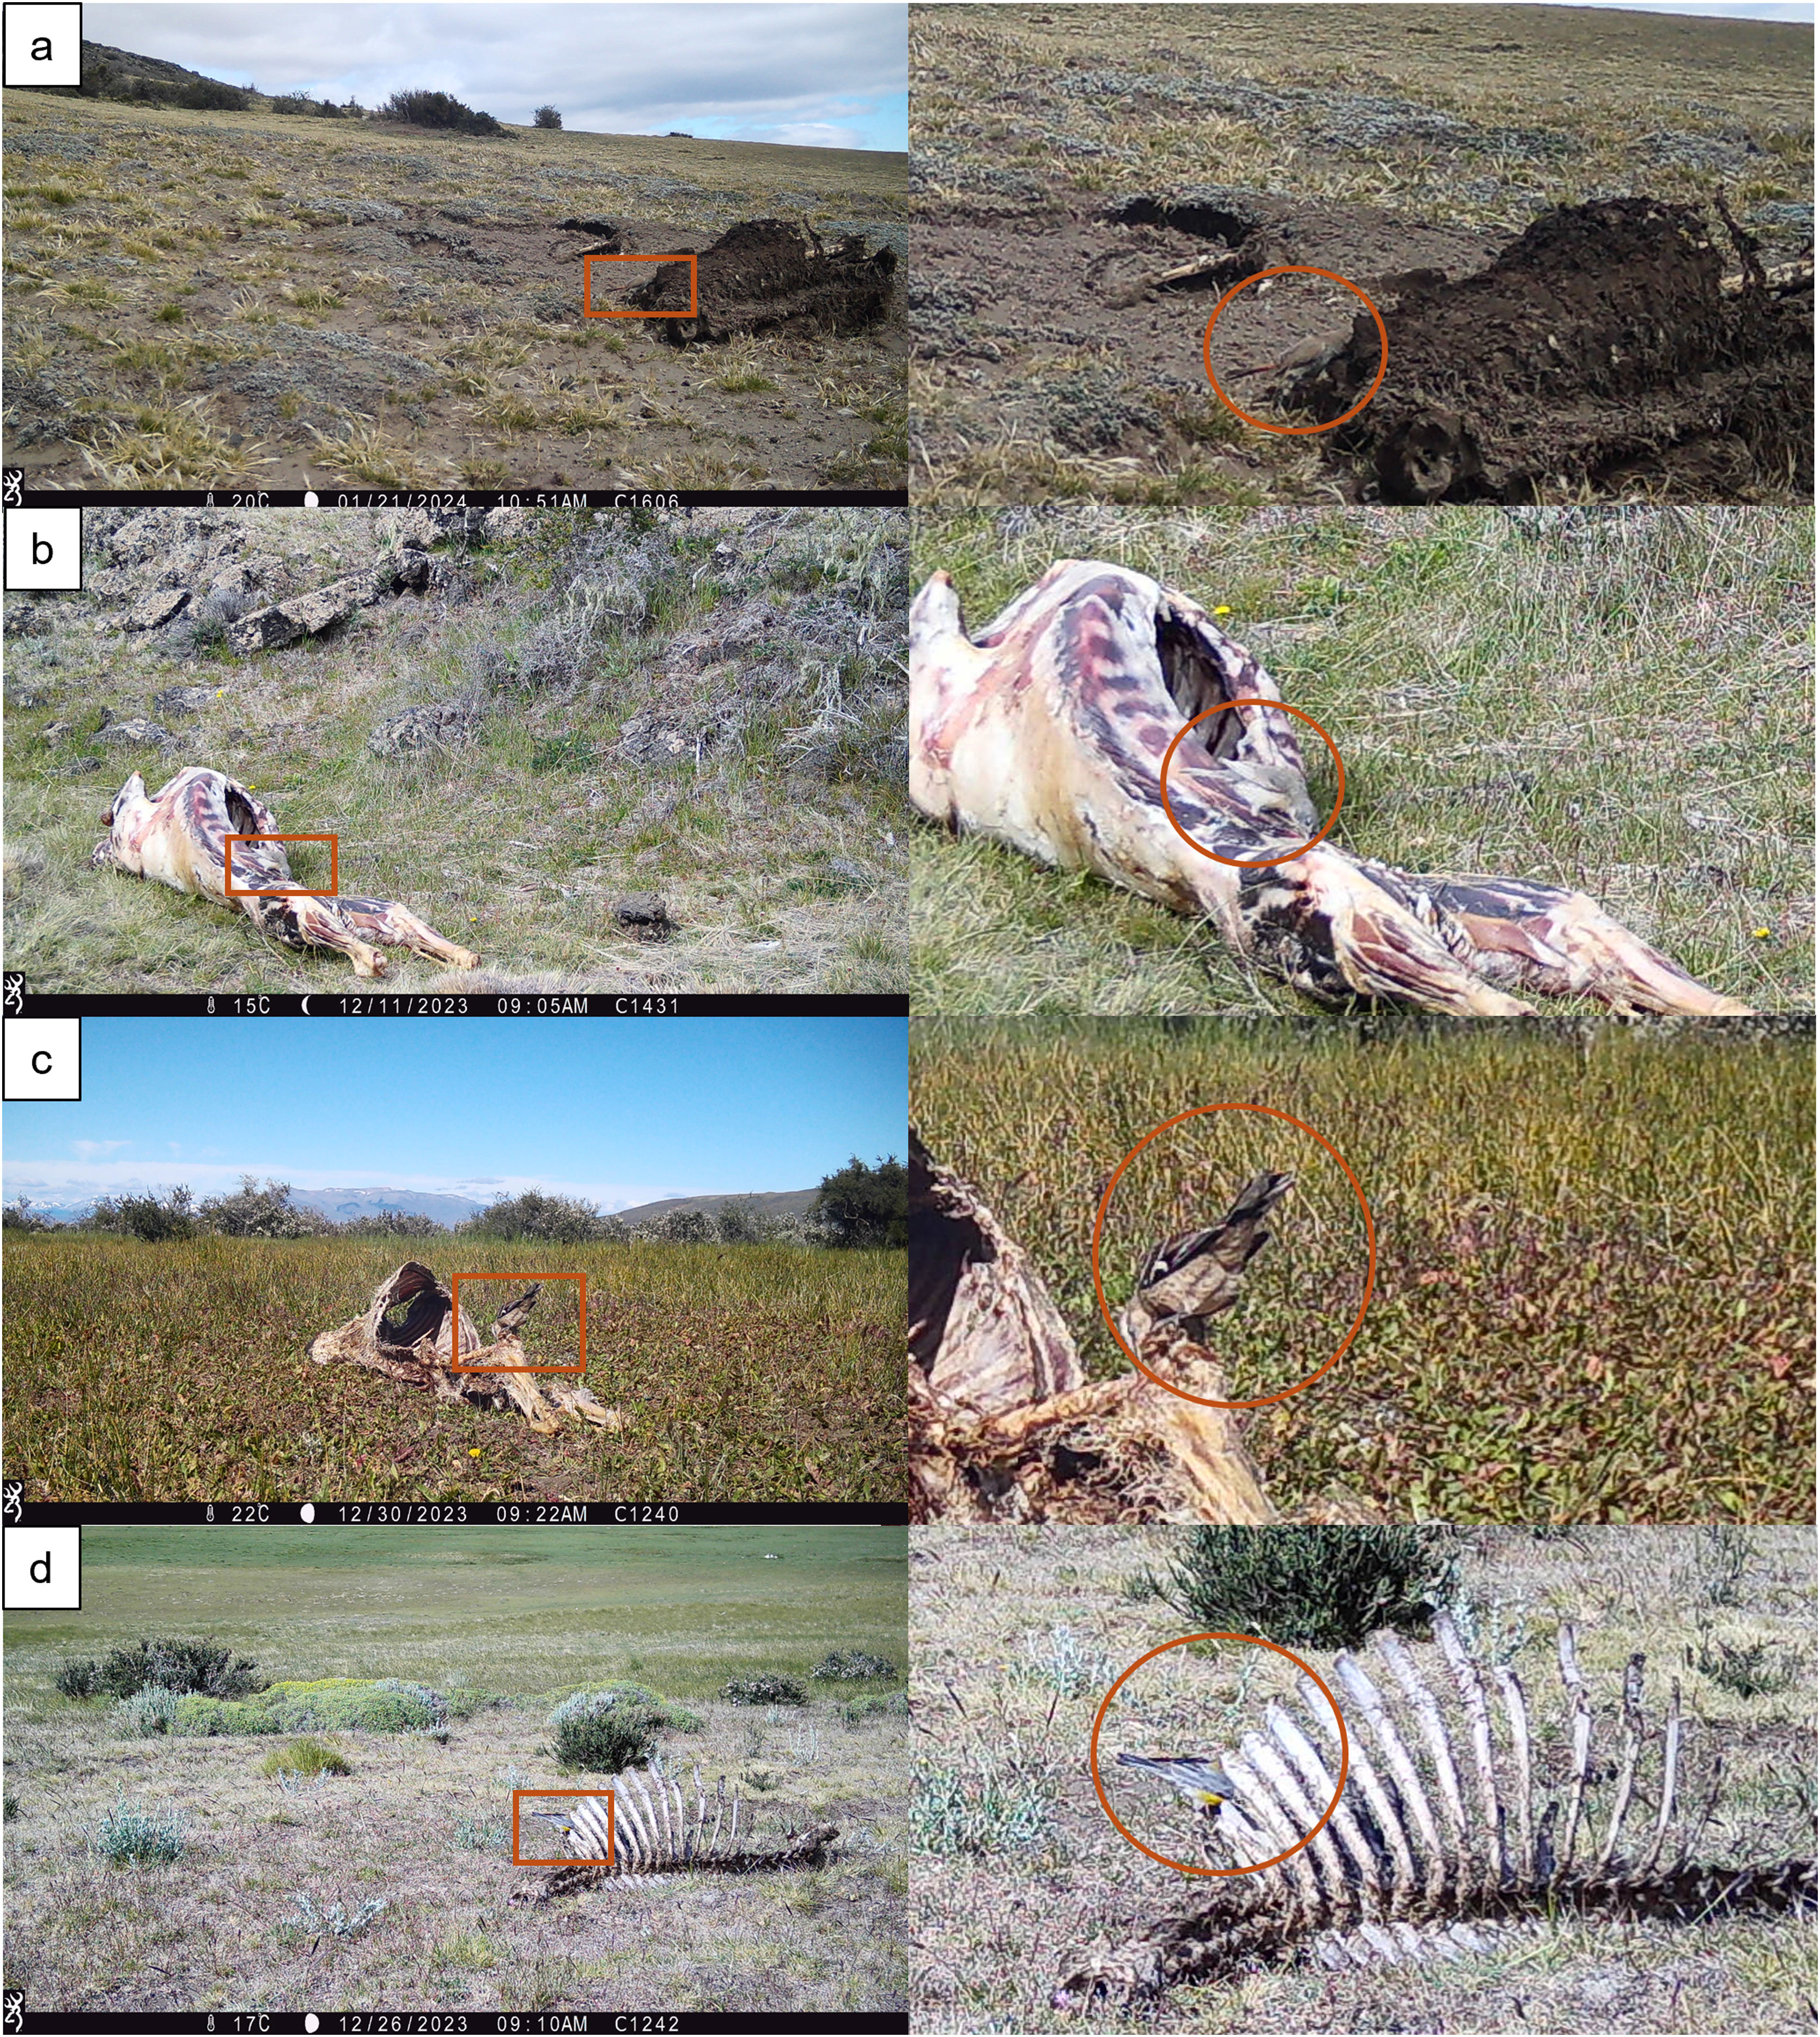
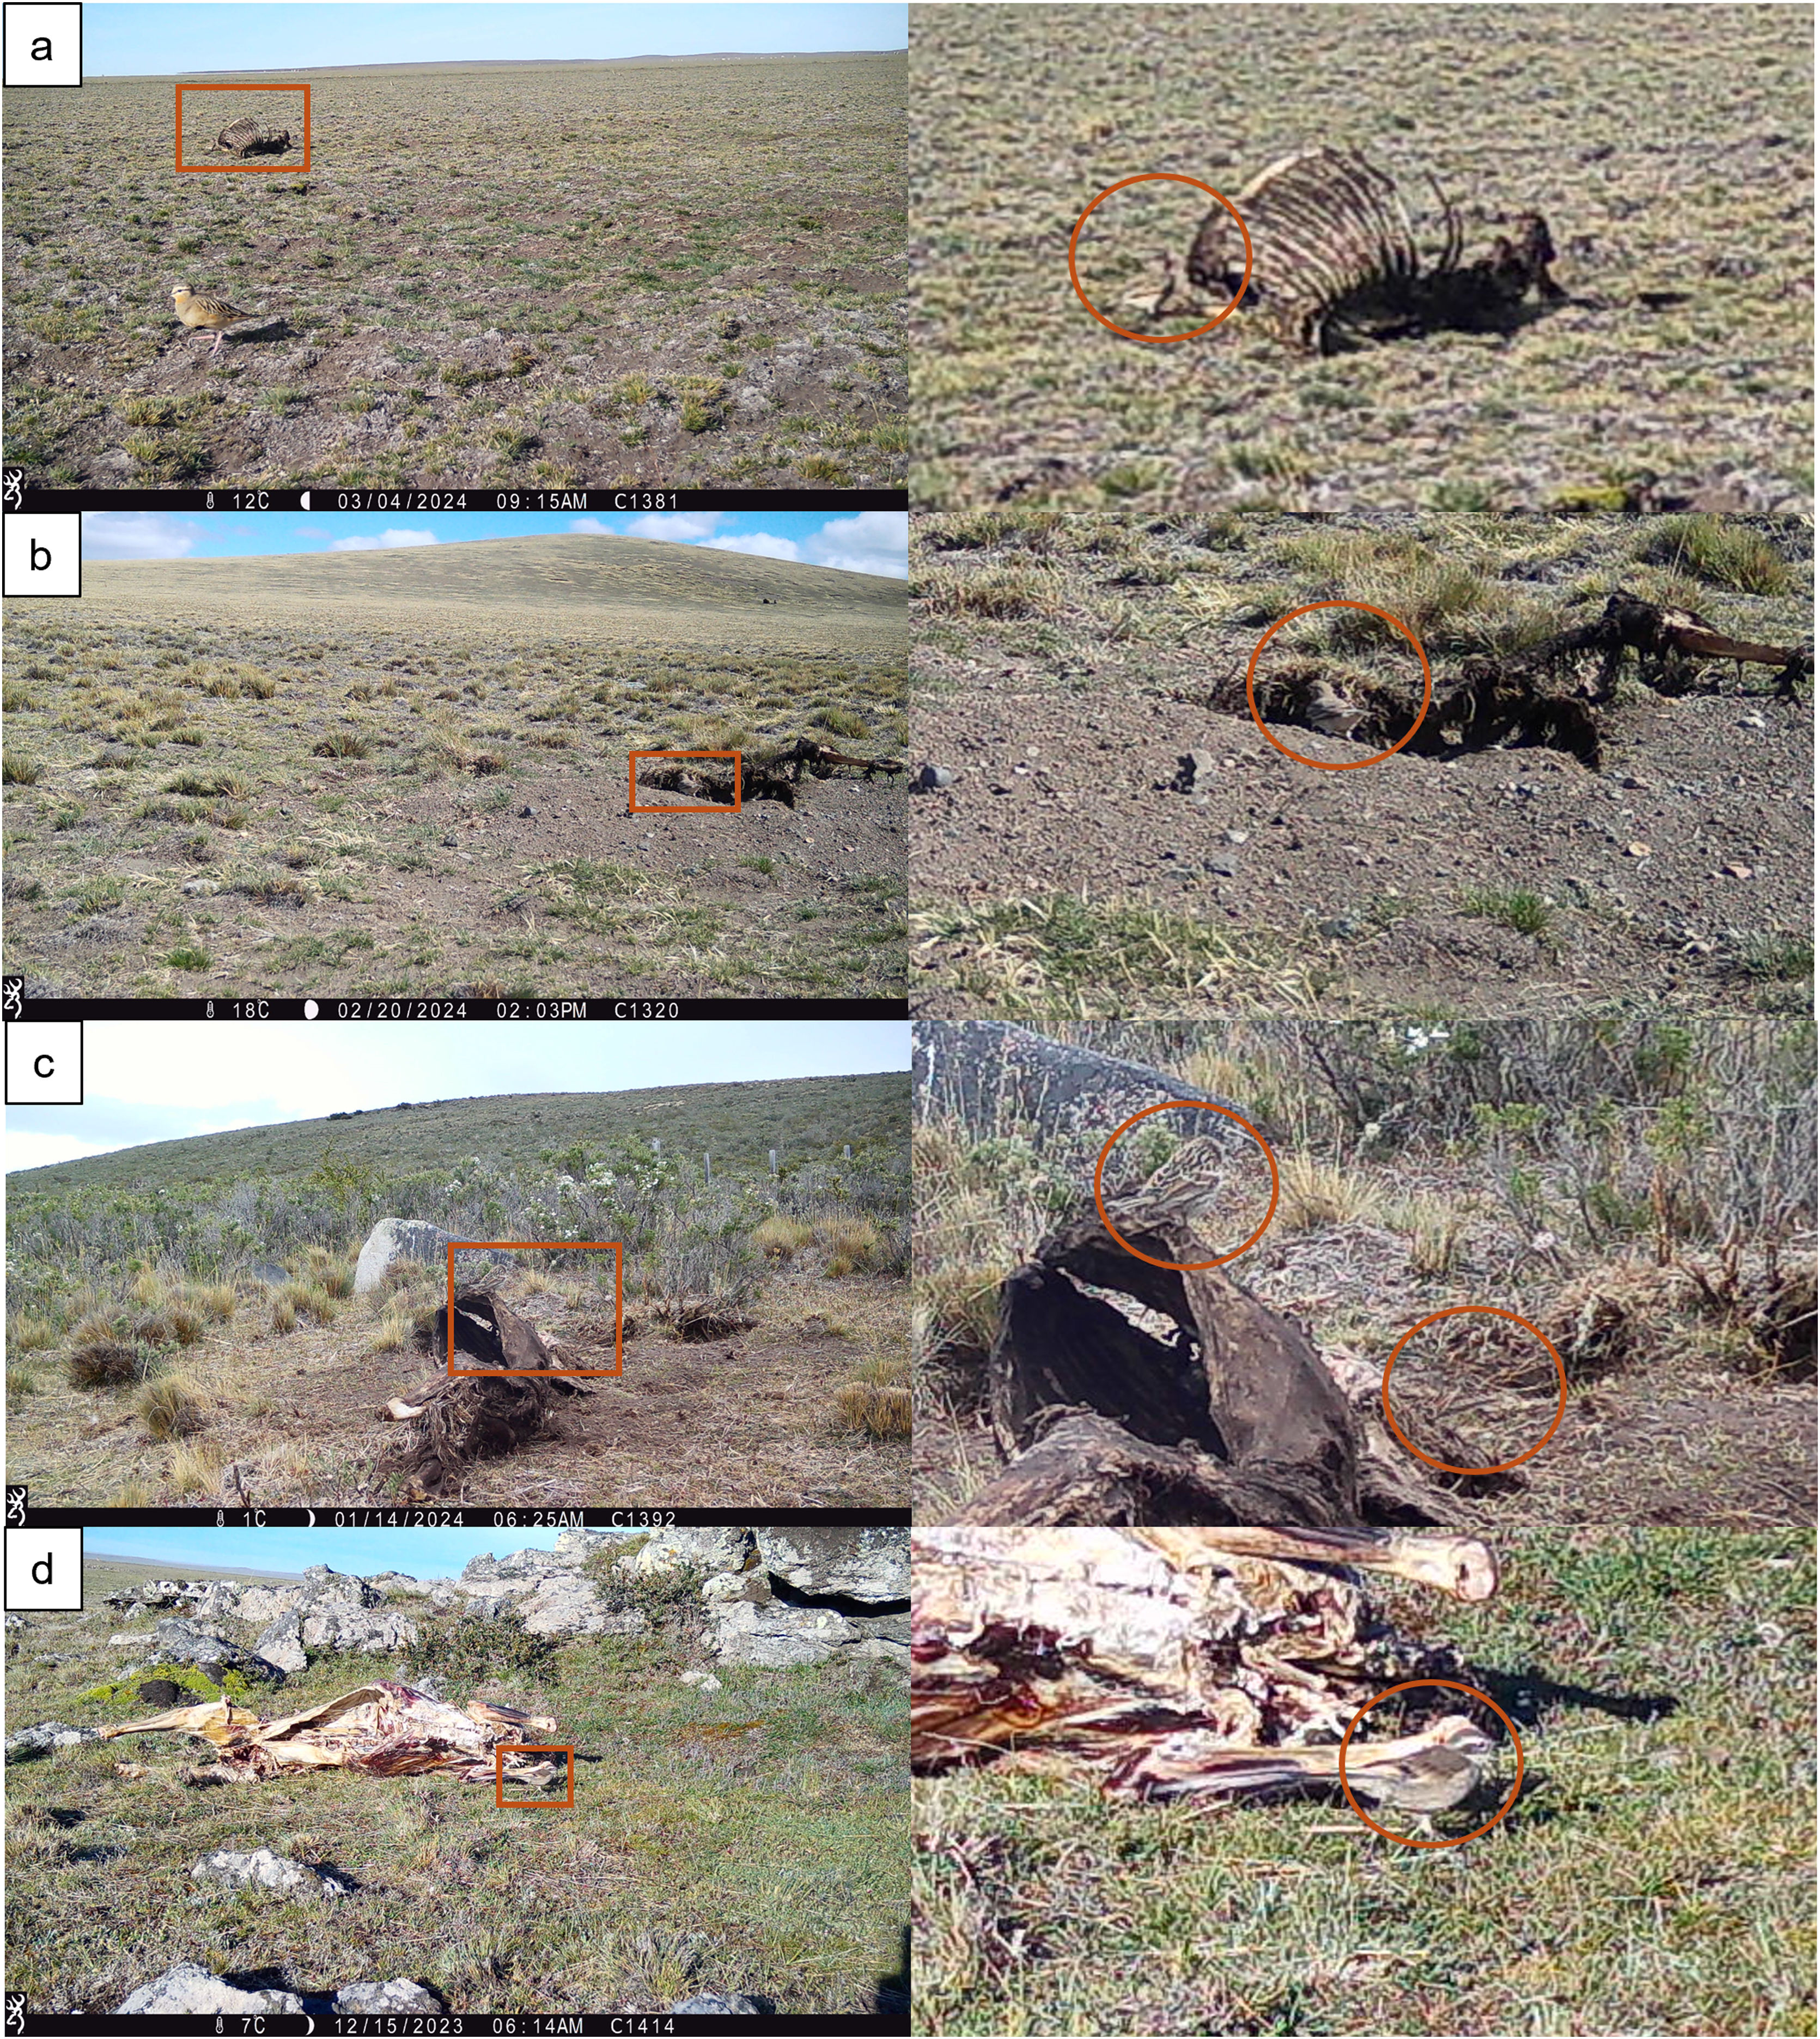
Carrion is a nutrient-rich yet unpredictable resource sustaining diverse vertebrate scavengers. We examined how environmental filters and species associations relate to scavenger guild structure under land-use change. In the Chilean Patagonian steppe, we deployed 70 ram carcasses across gradients of livestock management pressure, using a camera traps. At each carcass, we quantified species richness and a relative abundance index and applied Hill numbers (q = 0, 1, 2) to assess diversity, relating patterns to environmental variables and to large carnivores (puma Puma concolor and culpeo fox Lycalopex culpaeus) and dominant scavengers (Andean condor Vultur gryphus, grey fox L. griseus, kelp gull Larus dominicanus). We recorded 41 vertebrate species using carrion (i.e., interacting directly with carcass tissue or fluids), representing the highest richness reported for steppe ecosystems. Guild composition varied spatially, with facultative scavengers (kelp gulls, grey foxes) numerically replacing condors at some sites. Presence of puma and culpeo fox was associated with more even and diverse assemblages, whereas Andean condor and grey fox were associated with increased unevenness. These patterns suggest that species identity and livestock management are important correlates of scavenger community structure. Our findings provide a regional baseline for understanding how livestock management and large carnivore occurrence relate to carrion-mediated ecosystem processes.

Biological communities are structured by multiple interacting processes operating across spatial and temporal scales, including environmental filtering, interspecific interactions, and stochasticity (Mittelbach and Schemske, 2015). These processes determine community composition, ecosystem functioning, and ultimately the delivery of services such as nutrient cycling, pollination, and decomposition (Jacobs et al., 2013; Sebastián-González et al., 2020), which sustain life-supporting systems essential for human well-being (Andraczek et al., 2023). Understanding how these processes shape diversity patterns is therefore critical to maintaining ecosystem functioning and the human activities that depend on it.
Communities are not randomly assembled; their composition reflects filters acting at multiple scales (Mittelbach and Schemske, 2015). Processes such as drift, selection, speciation, and dispersal determine which species arrive and persist (Fukami, 2015; HilleRisLambers et al., 2012). Some species exert disproportionately strong influences on structure and function, either through dominance (high abundance or biomass; Avolio et al., 2019), or keystone effects (impacts exceeding abundance; Shukla et al., 2023). Recent frameworks emphasize that species roles, including dominance, apex trophic position, and keystone effects, emerge from interaction networks and should not be inferred solely from body size or trophic level without direct evidence of interaction-mediated influence (Inagaki et al., 2025). These mechanisms act simultaneously and interactively through space and time.
Among vertebrate communities, scavenger systems provide an exceptional model to examine assembly processes. Carrion represents a temporally and spatially discrete resource, where successional dynamics unfold rapidly as species detect, compete for, or facilitate access to carcasses under shifting abiotic conditions (Naves-Alegre et al., 2022). Such systems allow direct testing of non-neutral community assembly theory, where deterministic forces –environmental filtering, competition, and facilitation– drive structure and coexistence (Fukami, 2015; HilleRisLambers et al., 2012).
Carrion is not only a trophic resource but also a multifunctional ecological hotspot that supports a wide range of vertebrate interactions. Beyond direct consumption of carcass tissues, vertebrates may exploit carrion-associated resources in diverse ways, including ingestion of fluids, consumption of associated invertebrates, or use of materials such as hair and feathers (Moleón and Sánchez-Zapata, 2016; Redondo-Gómez et al., 2025). These interactions expand the ecological role of carrion beyond strict scavenging and highlight its importance as a resource integrating multiple trophic and non-trophic pathways within communities. Recognizing this broader spectrum of carrion use is essential for accurately characterizing the diversity and functional roles of vertebrates using carrion.
Within these systems, dominant and keystone species can strongly influence scavenger guild composition and function. Large obligate scavengers and apex predators shape carrion use by facilitating access (e.g., carcass opening) or excluding competitors (DeVault et al., 2003; Mateo-Tomás et al., 2017). These interactions determine both guild composition and carrion removal efficiency, a key ecosystem service, influencing nutrient redistribution and carcass decomposition dynamics (DeVault et al., 2003; Allen et al., 2015; Sebastián-González et al., 2021; Colino-Barea et al., 2026). Vultures (Cathartidae, Accipitridae) often dominate consumption through rapid detection and monopolizing, while large and medium carnivores may exert strong top-down effects within scavenger assemblages (Allen et al., 2015). Human-driven changes, such as livestock expansion, may disrupt these relationships (Mateo-Tomás et al., 2017).
Expanding food production has intensified livestock systems worldwide (Sadigov, 2022). Patagonia, with its extensive sheep ranching tradition (Radic-Schilling et al., 2024), provides a natural context to examine how such pressures affect vertebrate scavenger guild structure. Despite increasing global attention to scavenger ecology, little is known about how assembly mechanisms operate in relatively simple, open steppe ecosystems under sustained livestock management. Most research in southern South America has focused on avian scavenger or localized carcass studies, leaving unresolved how environmental filtering, dominance, and large carnivore presence interact to structure multispecies scavenger assemblages in Patagonian landscapes (Travaini et al., 1998; Cabrera-García et al., 2025). Evidence from other steppe systems suggests that top predators can strongly influence scavenger communities through both facilitative and risk-mediated effects (Perrig et al., 2023), a pattern that may be particularly evident in systems with relatively simple species pools (Sebastián-González et al., 2020), where facilitation and dominance interactions are more easily detected but may also increase vulnerability to environmental changes.
Here, we describe the structure of the vertebrate scavenger guild in the Patagonian steppe and evaluate how environmental filters and species associations relate to its diversity and composition. We focus on livestock management as a pervasive anthropogenic driver that alters vegetation structure, carcass size and habitat configuration, potentially acting as a non-random filter on scavenger communities (Bartel et al., 2023).
We hypothesize that scavenger diversity is associated with carcass size, livestock management pressure, and the presence of dominant and large apex carnivores. Specifically, we, predict that (1) larger carcasses are associated with higher diversity; (2) increasing livestock management intensity is associated with reduced scavenger diversity through environmental filtering; and (3) carcasses characterized by dominance or large carnivore presence differ in diversity and composition patterns consistent with facilitation or competitive structuring.
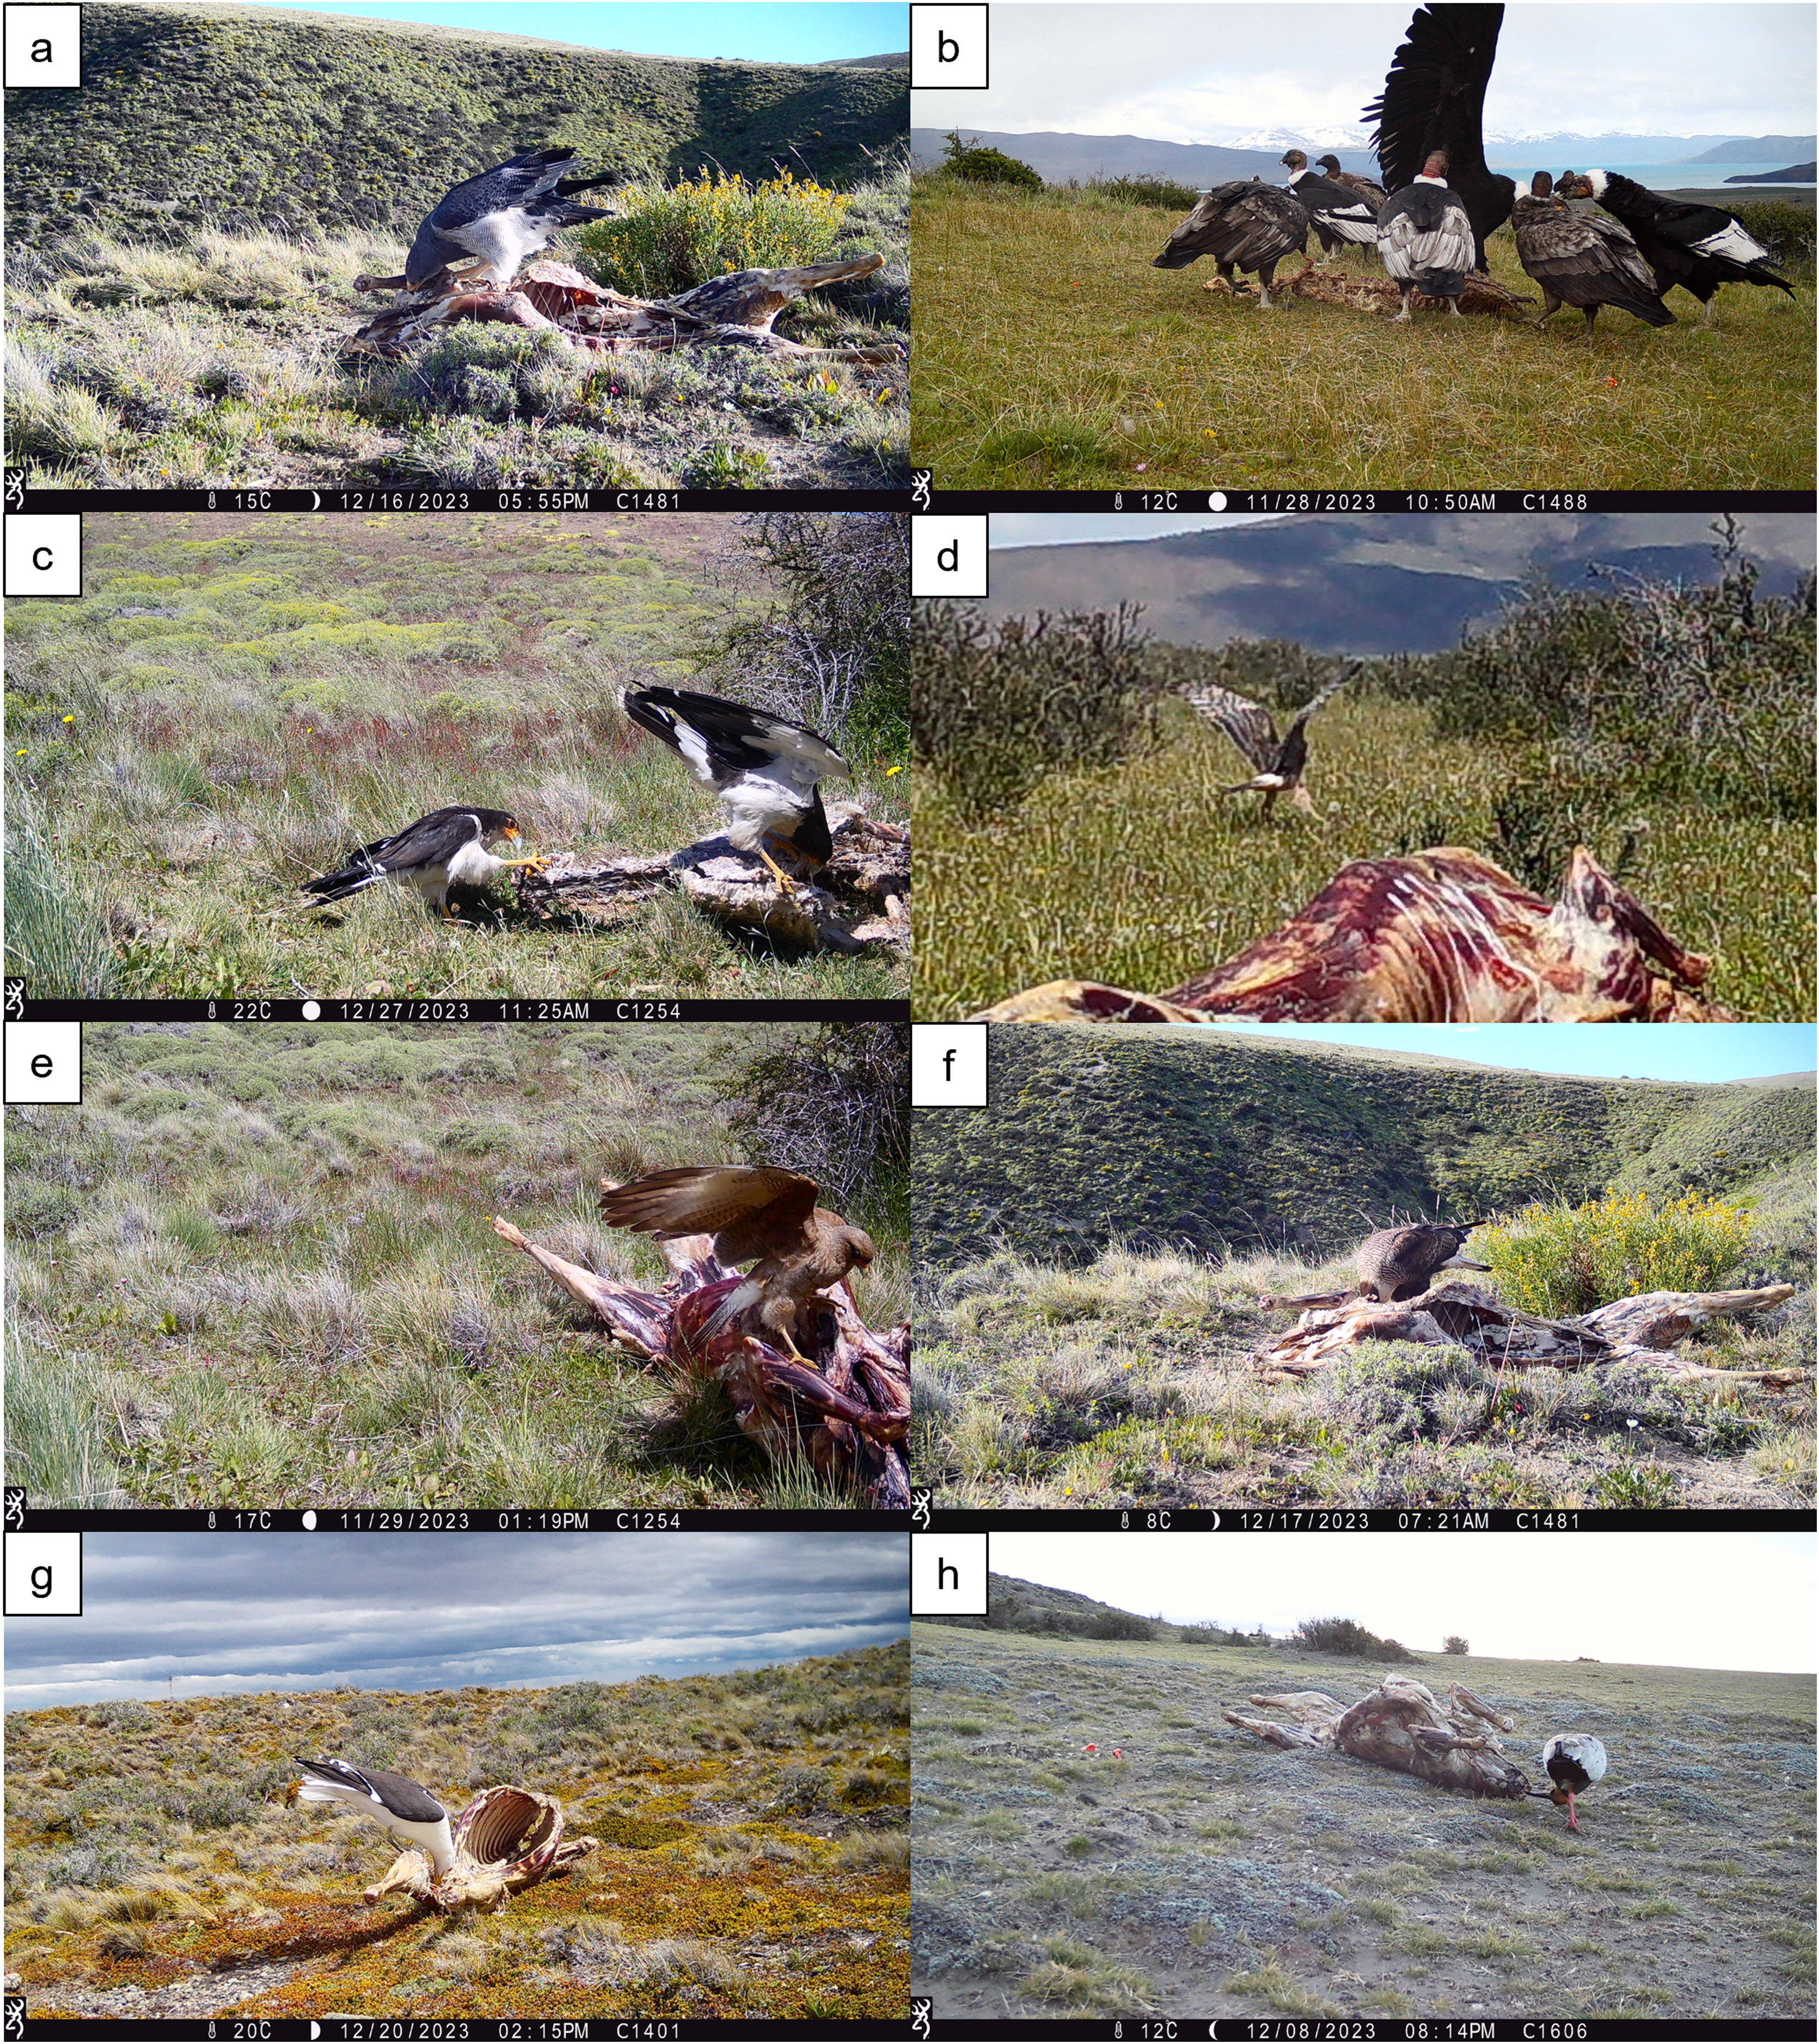
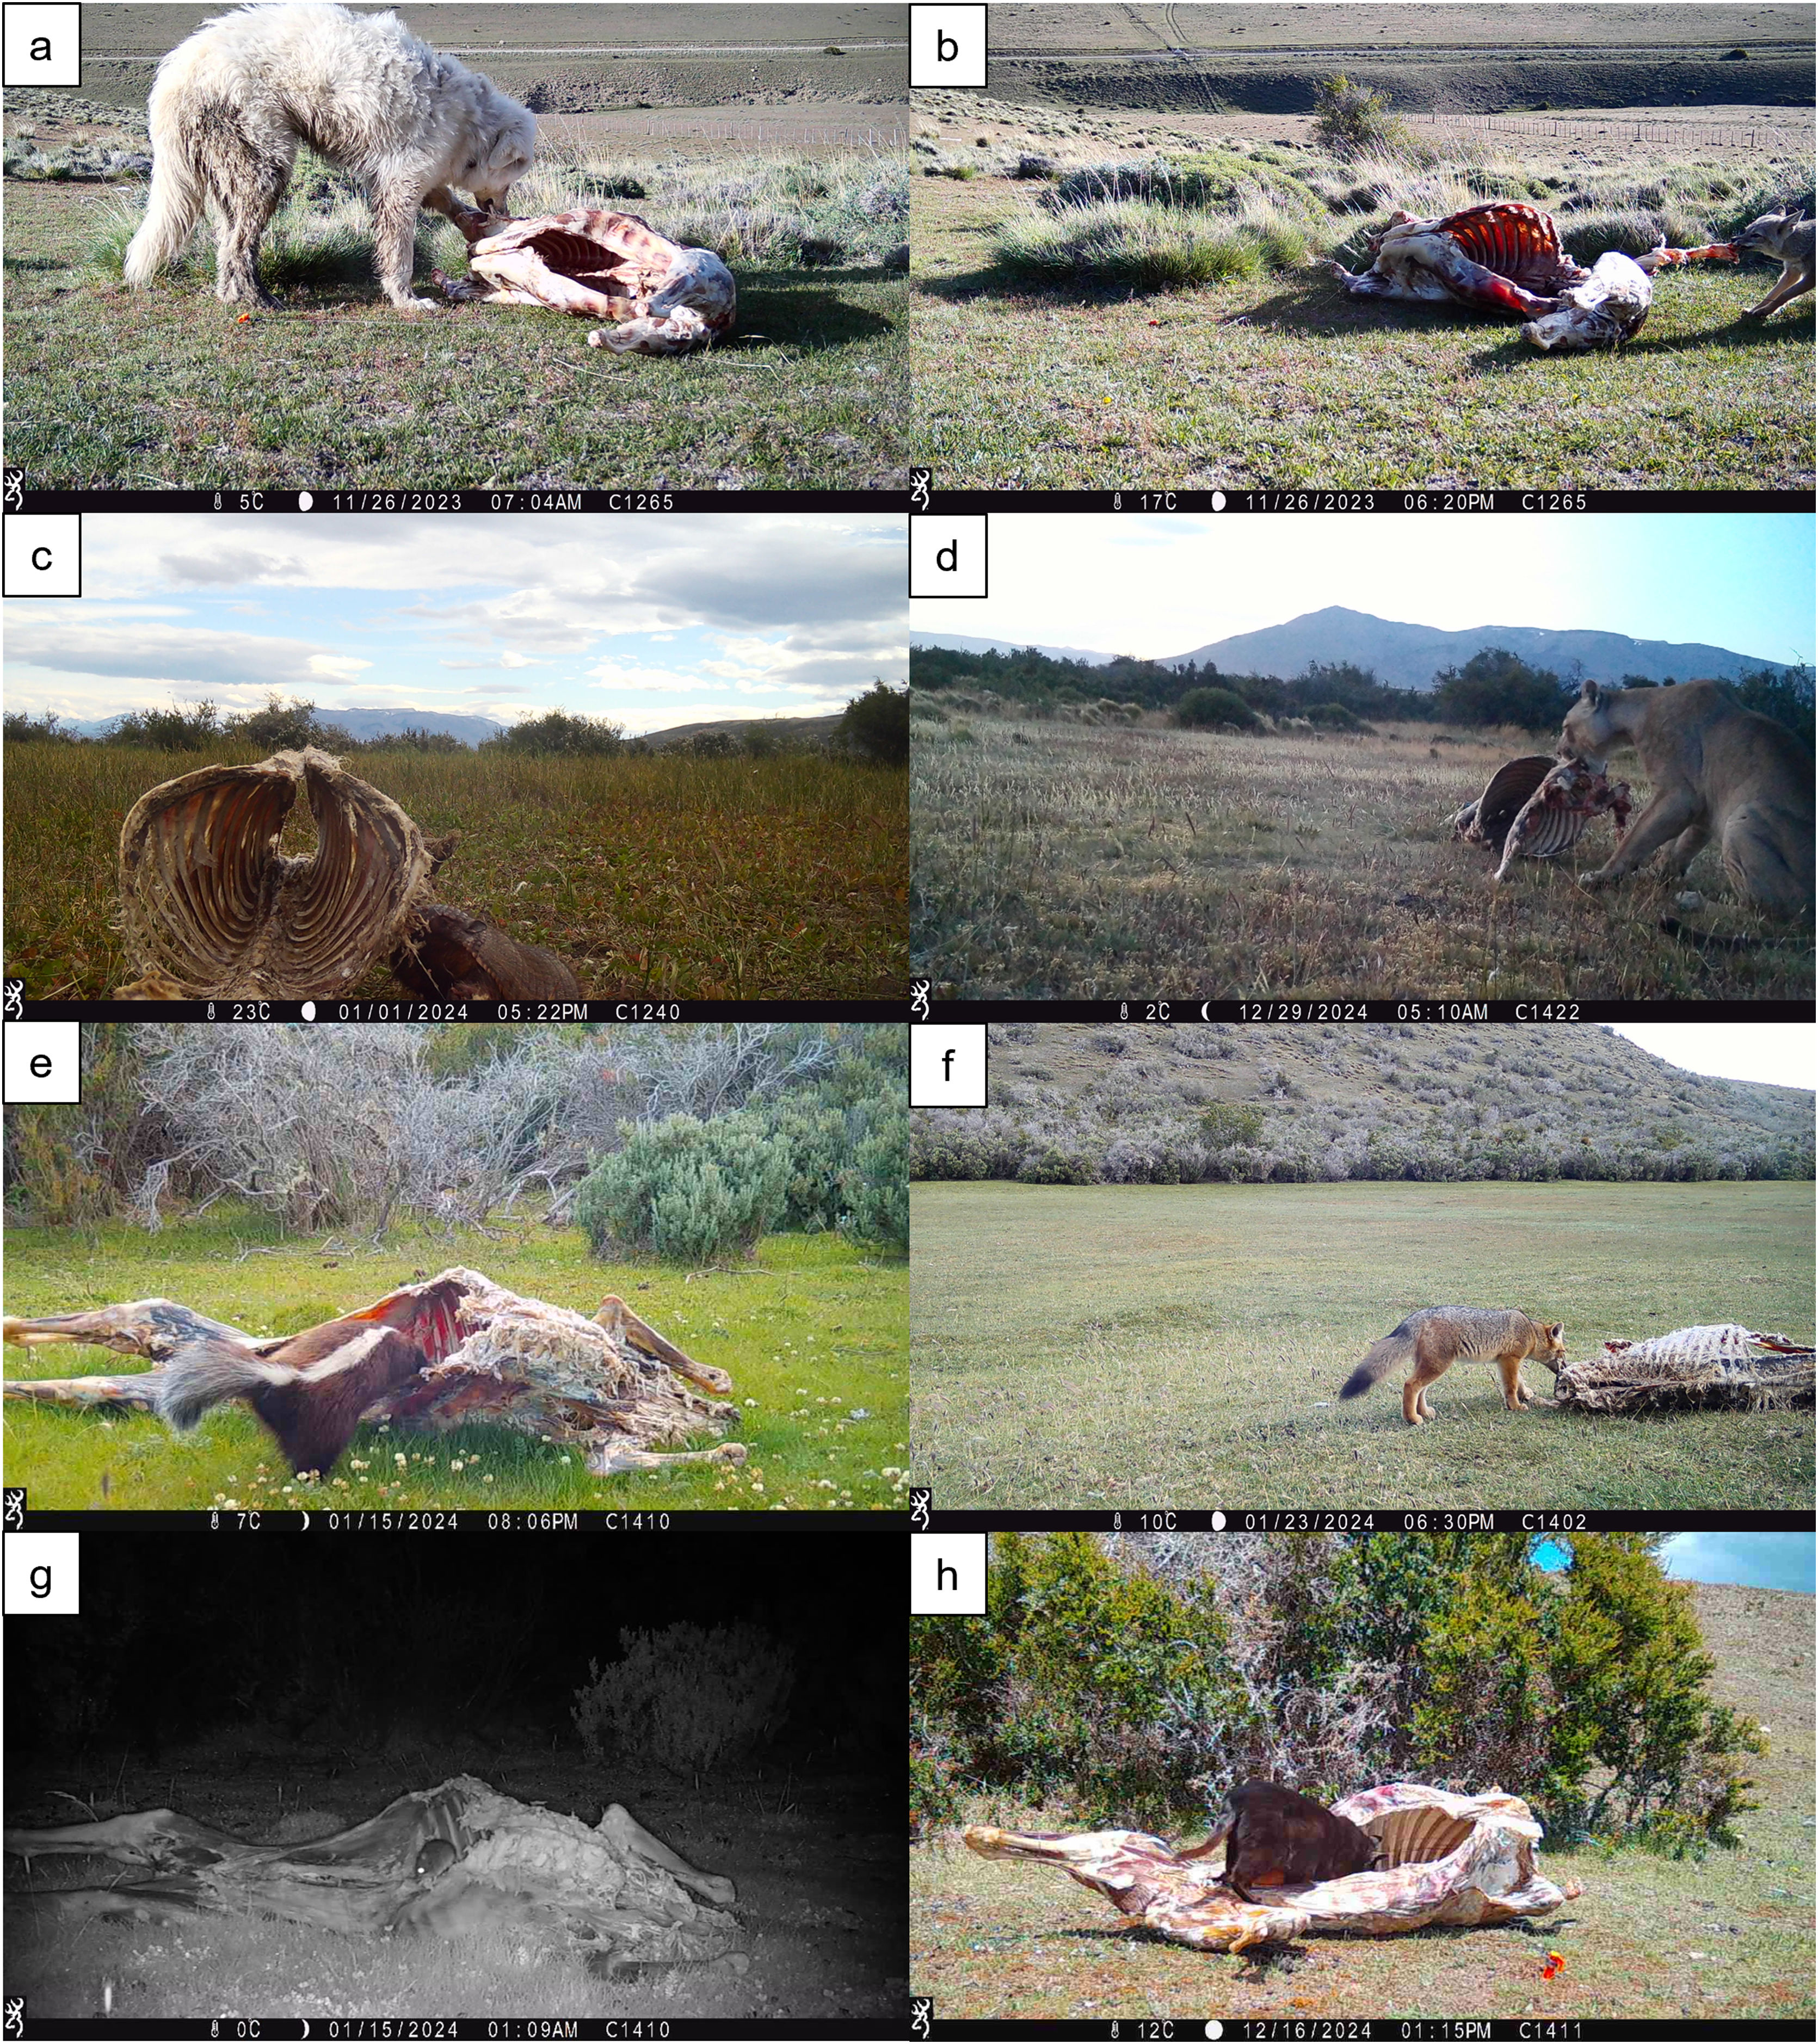
Material and methodsStudy site and species presenceThe research was conducted in the Magallanes District, southern Chile, in the provinces of Última Esperanza (ULT; 50°47′S, 74°06′W) and Magallanes (MAG; 53°10′S, 70°56′W; Fig. 1). Three sites were selected in each province: one national park and two livestock ranches. In ULT, these were Torres del Paine National Park (TPNP) and CG (≈ 2.2 sheep/ha) and RN (≈ 0.2 sheep/ha) ranches; in MAG, Pali-Aike National Park (PANP) and LP (≈ 0.2 sheep/ha) and JO (≈ 0.7 sheep/ha) ranches. Reported values correspond to instantaneous stocking densities calculated at the paddock level and restricted to paddocks actively grazed at the time of sampling (i.e., empty paddocks were excluded). Sheep numbers ranged from ca. 3,000 and 5,000 per ranch. Guanacos (Lama guanicoe) co‐occurred with sheep at CG and LP and were also present in both national parks. Sites represented a gradient of livestock management pressure: I) none (TPNP and PANP, guanacos only); II) medium (CG and LP, guanacos and sheep); and III) high (RN and JO, sheep only). Livestock management pressure categories were defined based on management regime and tolerance to native wildlife (i.e., co-occurrence with guanacos), rather than stocking density alone. In this context, medium-pressure sites allow the coexistence of livestock and native herbivores, whereas high-pressure sites are characterized by exclusive livestock use and reduced tolerance to wildlife. All sites lie within the Patagonian steppe, which is dominated by tussock grass (Festuca gracillima), with summer temperatures near 10 °C, winter means of 0−3 °C, and annual precipitation of 200–588 mm, mostly snow (Radic-Schilling et al., 2024). This ecosystem supports three obligate scavengers –Andean condor (Houston et al., 2020), black vulture (Coragyps atratus; Buckley et al., 2022), and turkey vulture (Cathartes aura; Kirk and Mossman, 2020)– and various facultative scavengers including culpeo fox, Patagonian hog-nosed skunk (Conepatus humboldtii), caracaras (i.e., crested Caracara plancus, chimango Daptrius chimango, white-throated Daptrius albogularis), raptors (e.g., black-chested buzzard-eagle Geranoaetus melanoleucus), passerines (e.g., thorn-tailed rayadito Aphrastura spinicauda), and lizards (Liolaemus spp.) all documented exploiting carrion or predator-provided carcasses in Patagonia (Elbroch and Wittmer, 2012; Jaksic et al., 2002).
Experimental design and data sampling
During late spring-early summer 2023 (November-December, southern hemisphere), we deployed 70 ram carcasses across the six sites spanning the full gradient of livestock management pressure. All carcasses were installed within the same week and monitored simultaneously throughout the study period. Ten carcasses were placed at each no-pressure and high-pressure site (TPNP, PANP, RN, JO) and 15 in each moderate-pressure site (CG, LP).
Each carcass was monitored using a single motion-activated camera trap (Browning Strike Force Cam, Birmingham, AL) programmed to capture three photographs per motion event with a 5-s delay between triggers. Carcasses, obtained from a certified slaughterhouse, were anchored to the ground within the camera’s field of view. The first carcass at each site was placed at a randomly location, and subsequent units were installed ≥ 1 km apart whenever terrain and access permitted.
Carcasses were monitored continuously from deployment until complete depletion or removal from the camera’s field of view by scavengers. The research activities were conducted under authorisation from the Chilean National Forestry Service (CONAF; permits No. 155/2023 and 121/2024) for work within national parks. Landowners granted permission to access and conduct fieldwork on private ranches. All activities procedures complied with national and institutional regulations and were approved by the Bioethics Committee of the University Austral of Chile (Ref. No. 493/2023).
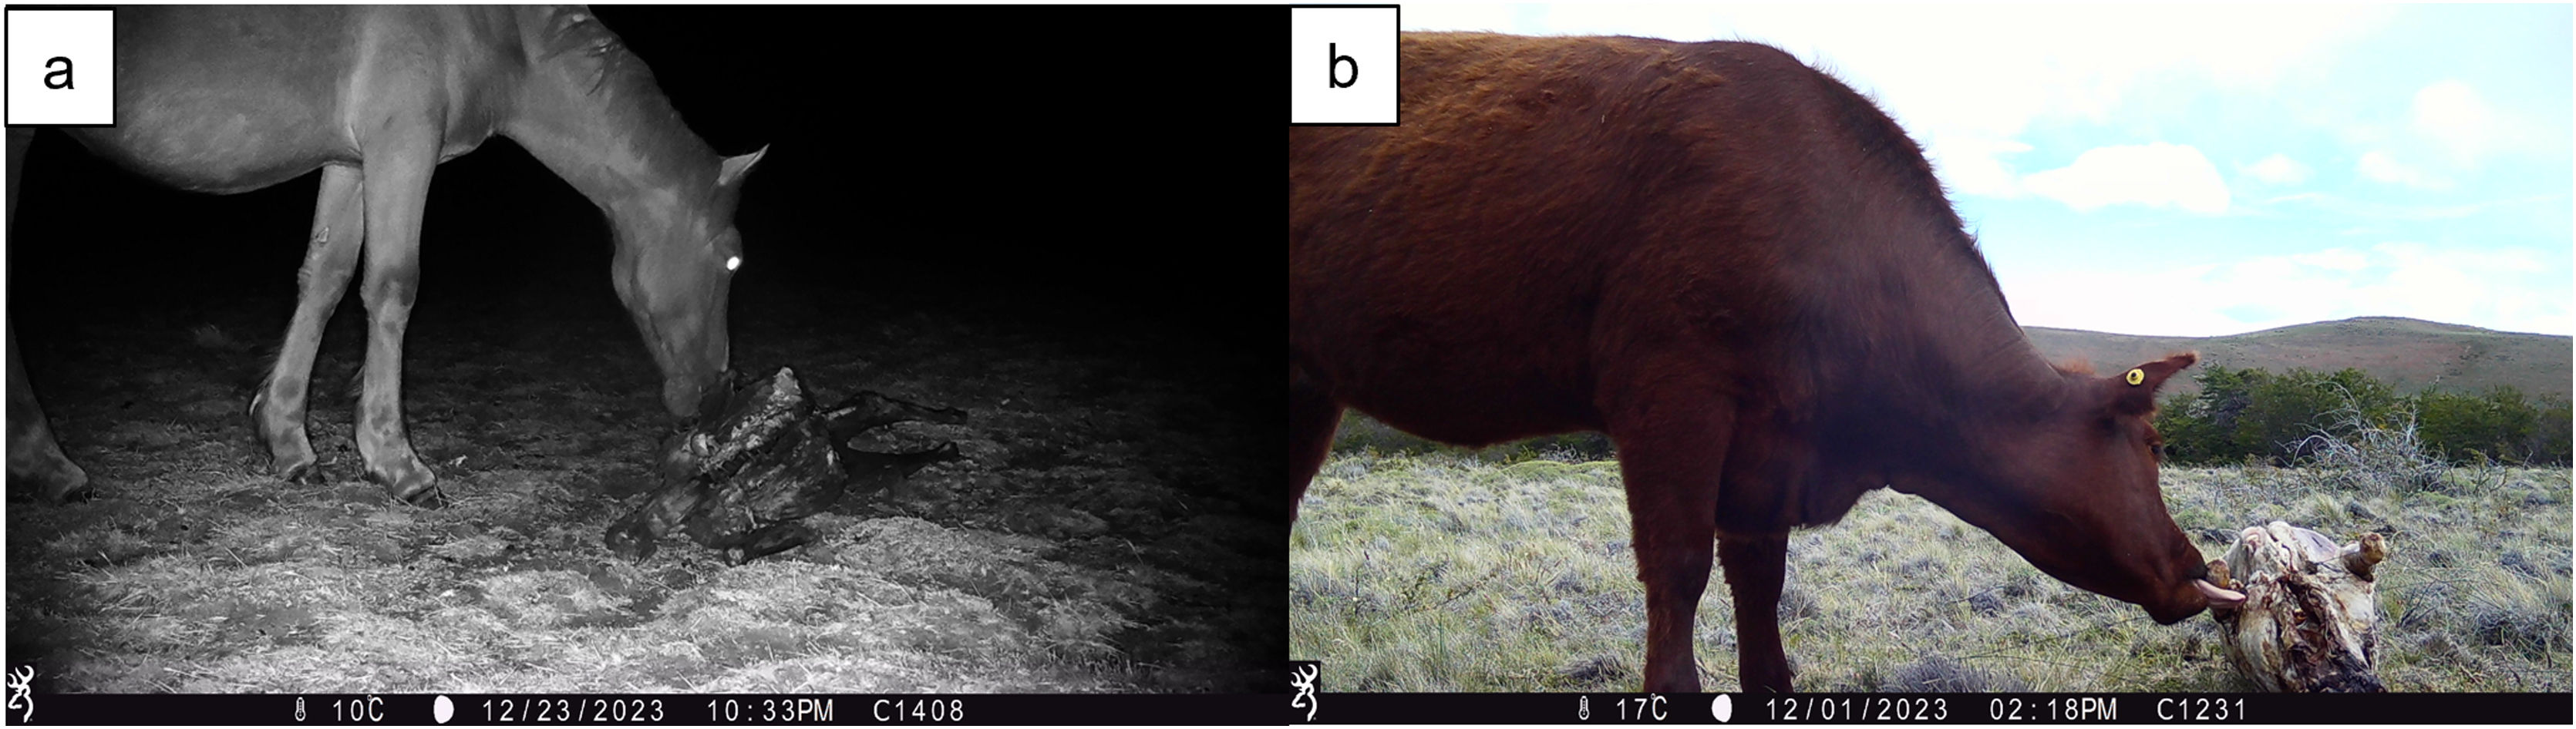
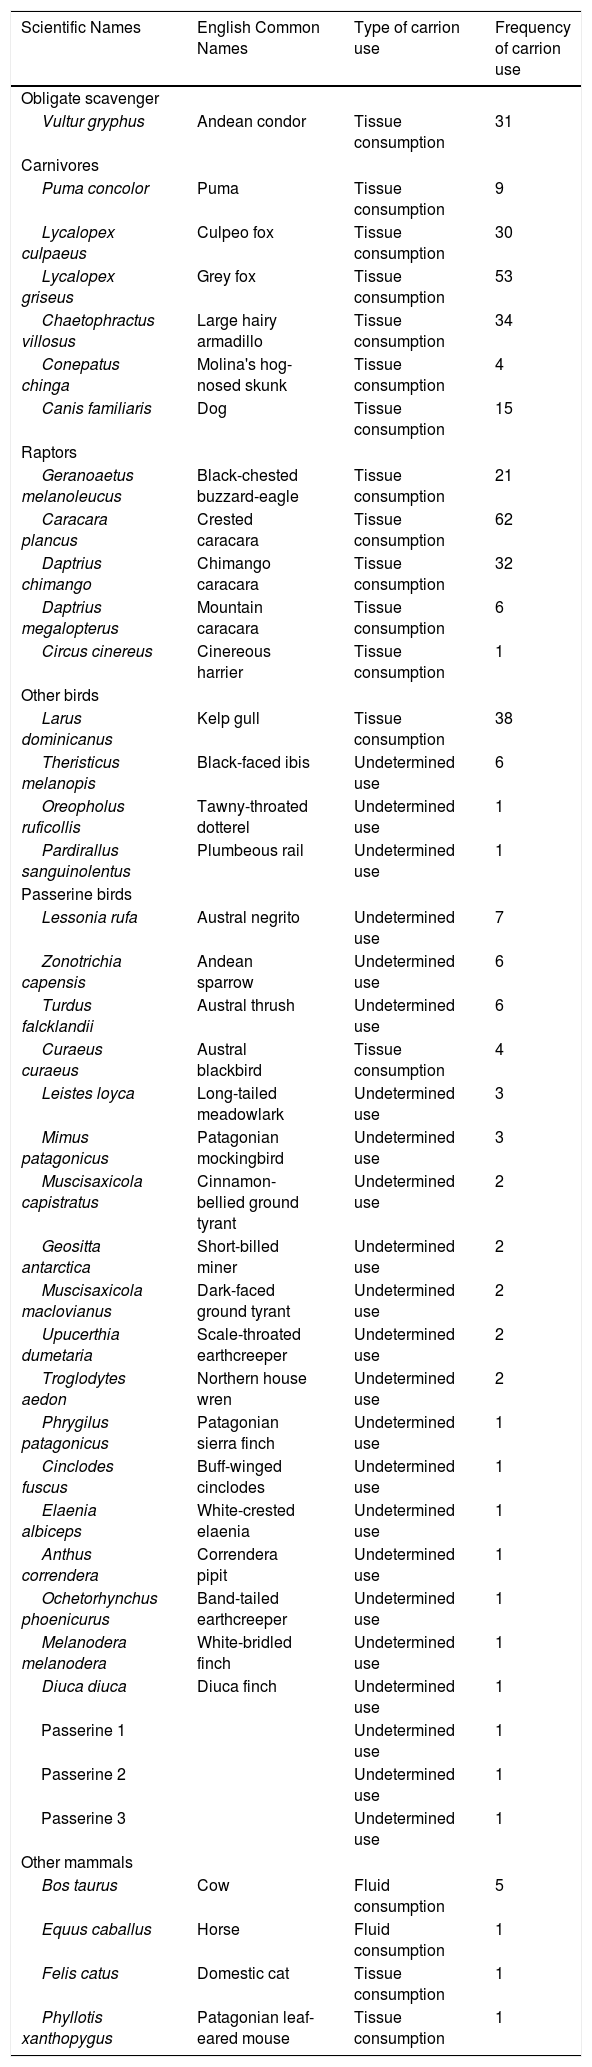
Scavenging metrics and data analysisAll images were manually reviewed in three rounds by an observer experienced in camera-trap data analyses and local species identification. For each carcass, we recorded two metrics: species richness and a relative abundance index. Species richness was defined as the number of vertebrate species showing direct interaction with carcass tissue or fluids. These interactions were classified according to type of carrion use, including tissue consumption (direct observation of pecking, tearing, or biting), fluid consumption (e.g., licking of carcass-derived fluids), and undetermined use based on behavioural posture consistent with feeding but without clear visual confirmation of tissue ingestion (Table 1). Species merely present near carcasses without visible tissue contact were not considered as using carrion. The relative abundance index was defined as the maximum number of individuals of a given species simultaneously visible in an image or, when distinguishable, the cumulative number of individuals identified based on age, sex, or body size. As detection probability may vary among taxa, this metric represents a detection-based index rather than true population abundance and may be influences by species-specific traits such as body size, conspicuousness, group size, and behavioural patterns. These data were used to construct a carcass-by-species abundance matrix (Leibold and Mikkelson, 2002).
Vertebrate species recorded using carrion at experimental carcasses in the Chilean Patagonian steppe. Species are grouped by functional and taxonomic categories. For each species, we report scientific and common names, type of carrion use, and frequency of occurrence, defined as the number of carcasses (out of 70) at which individuals were observed directly interacting with carcass tissue or fluids. Carrion use was classified as: tissue consumption (direct evidence of pecking, tearing, or biting), fluid consumption (licking or ingestion of carcass-derived fluids), and undetermined use (behaviour consistent with feeding but without clear visual confirmation of tissue ingestion). Unidentified passerines (“Passerine 1–3”) correspond to individuals that could not be reliably assigned to species level from camera-trap images.
| Scientific Names | English Common Names | Type of carrion use | Frequency of carrion use |
|---|---|---|---|
| Obligate scavenger | |||
| Vultur gryphus | Andean condor | Tissue consumption | 31 |
| Carnivores | |||
| Puma concolor | Puma | Tissue consumption | 9 |
| Lycalopex culpaeus | Culpeo fox | Tissue consumption | 30 |
| Lycalopex griseus | Grey fox | Tissue consumption | 53 |
| Chaetophractus villosus | Large hairy armadillo | Tissue consumption | 34 |
| Conepatus chinga | Molina's hog-nosed skunk | Tissue consumption | 4 |
| Canis familiaris | Dog | Tissue consumption | 15 |
| Raptors | |||
| Geranoaetus melanoleucus | Black-chested buzzard-eagle | Tissue consumption | 21 |
| Caracara plancus | Crested caracara | Tissue consumption | 62 |
| Daptrius chimango | Chimango caracara | Tissue consumption | 32 |
| Daptrius megalopterus | Mountain caracara | Tissue consumption | 6 |
| Circus cinereus | Cinereous harrier | Tissue consumption | 1 |
| Other birds | |||
| Larus dominicanus | Kelp gull | Tissue consumption | 38 |
| Theristicus melanopis | Black-faced ibis | Undetermined use | 6 |
| Oreopholus ruficollis | Tawny-throated dotterel | Undetermined use | 1 |
| Pardirallus sanguinolentus | Plumbeous rail | Undetermined use | 1 |
| Passerine birds | |||
| Lessonia rufa | Austral negrito | Undetermined use | 7 |
| Zonotrichia capensis | Andean sparrow | Undetermined use | 6 |
| Turdus falcklandii | Austral thrush | Undetermined use | 6 |
| Curaeus curaeus | Austral blackbird | Tissue consumption | 4 |
| Leistes loyca | Long-tailed meadowlark | Undetermined use | 3 |
| Mimus patagonicus | Patagonian mockingbird | Undetermined use | 3 |
| Muscisaxicola capistratus | Cinnamon-bellied ground tyrant | Undetermined use | 2 |
| Geositta antarctica | Short-billed miner | Undetermined use | 2 |
| Muscisaxicola maclovianus | Dark-faced ground tyrant | Undetermined use | 2 |
| Upucerthia dumetaria | Scale-throated earthcreeper | Undetermined use | 2 |
| Troglodytes aedon | Northern house wren | Undetermined use | 2 |
| Phrygilus patagonicus | Patagonian sierra finch | Undetermined use | 1 |
| Cinclodes fuscus | Buff-winged cinclodes | Undetermined use | 1 |
| Elaenia albiceps | White-crested elaenia | Undetermined use | 1 |
| Anthus correndera | Correndera pipit | Undetermined use | 1 |
| Ochetorhynchus phoenicurus | Band-tailed earthcreeper | Undetermined use | 1 |
| Melanodera melanodera | White-bridled finch | Undetermined use | 1 |
| Diuca diuca | Diuca finch | Undetermined use | 1 |
| Passerine 1 | Undetermined use | 1 | |
| Passerine 2 | Undetermined use | 1 | |
| Passerine 3 | Undetermined use | 1 | |
| Other mammals | |||
| Bos taurus | Cow | Fluid consumption | 5 |
| Equus caballus | Horse | Fluid consumption | 1 |
| Felis catus | Domestic cat | Tissue consumption | 1 |
| Phyllotis xanthopygus | Patagonian leaf-eared mouse | Tissue consumption | 1 |
From this matrix, we aggregated data by summing abundances across carcasses within each site, generating a site-by-species matrix. We then estimate alpha-diversity using Hill numbers, where q = 0 corresponds to species richness, q = 1 corresponds to Shannon diversity, and q = 2 corresponds to Simpson diversity, following Chao et al. (2014). Because Hill numbers increasingly weight species according to their relative abundance, q = 1 is sensitive to species evenness, whereas q = 2 is more influenced by dominant species. Diversity estimates were computed using the iNEXT R package (Hsieh et al., 2016), applying individual-based rarefaction and extrapolation using the number of detected individuals as the sampling unit. This approach allows standardized comparison of diversity among assemblages with unequal detection frequencies (Chao et al., 2014). To visualize carcass-level community composition, we generate a heatmap of relative species abundance per carcass. Gamma diversity was calculated as the total number of species observed across all sites, and beta diversity as the ratio of gamma to mean alpha diversity (Oksanen et al., 2020). Dominance was evaluated at the carcass level, with species exceeding 30% of the relative abundance index considered dominant within that assemblage. This cutoff was applied as a pragmatic criterion to identify disproportionate contributions, recognizing that dominance is context-dependent (Avolio et al., 2019). Large apex carnivores (e.g., puma and culpeo fox) were analysed separately due to their trophic position and potential to influence scavenger interactions and carrion access, consistent with interaction-based frameworks describing species roles in scavenger assemblages (Shukla et al., 2023; Inagaki et al., 2025).
We analysed carcass-level composition using RDA of Hellinger-transformed carcass-by-species abundances. Predictors included province (MAG, ULT), livestock management pressure (none/medium/high), vegetation cover (within 3 m radius), initial carcass mass, carcass duration, and the province-by-pressure interaction. Continuous variables were standardized, and carcass duration was log10(x+1)-transformed. Model, terms, and axis significance were tested with 999 permutations, and ordinations are shown with a scaling-2 biplot. Given a significant overall pressure effect, we performed pairwise PERMANOVA (Bray-Curtis) using vegan 2.7−1 (Oksanen et al., 2020) and pairwiseAdonis (Martinez Arbizu, 2020).
To identify drivers of the diversity of vertebrates using carrion (Hill q = 0, 1, 2) at the carcass level, we used an information-theoretic approach with exhaustive model selection a nonparametric bootstrapping. Candidate models represented three ecological mechanisms: (i) dominant scavengers (Andean condor, grey fox, kelp gull), (ii) Large apex carnivores (puma, culpeo fox), (iii) and environment (livestock management pressure, vegetation cover, initial carcass mass, carcass duration, province). Eleven hypotheses were tested: H0 (Null), H1 (carcass duration), H2 (province), H3 (environment), H4 (full environment), H5 (Apex), H6 (dominants), H7 (hierarchy), H8 (environment + apex), H9 (environment + dominants), H10 (Full).
We modelled q = 0 with Conway-Maxwell-Poisson GLMs and q = 1, 2 with Gamma GLMs. Models were ranked by AICc; ΔAICc <2 defined supported sets (Burnham and Anderson, 2002). Within each 500 bootstrap iterations, we computed model-averaged coefficients and unconditional variable importance. Effects were considered significant when 95% percentile CIs excluded zero (Nakagawa and Cuthill, 2007) and are reported as multiplicative changes relative to baselines.
ResultsA total of 3,816 trap-days yielded 973,445 images across the 70 monitored carcasses. Monitoring lasted 5–109 days per carcass (mean ± SD = 54.5 ± 31.5). Site-level richness (q = 0) ranged from 13 to 20 species (Fig. 2a, b). Total gamma-diversity across all sites was 41 vertebrate species using carrion (Figs. 3a, S1–S9; Table 1), yielding beta = 2.59, indicating moderate turnover. Accounting for abundances revealed declining diversity and increasing unevenness: q = 1 ranged 5.86–10.73 and q = 2 3.58–7.83 (Fig. 2c-f). The steepest drops from q = 0 to q = 2 occurred at PANP and LP (strong dominance), whereas JO and TPNP showed higher evenness, with CG and RN intermediate.

Rarefaction and extrapolation curves of alpha diversity across sampling sites in the two provinces, based on Hill numbers. Panels show diversity patterns for ULT and MAG provinces. The x-axis represents the cumulative number of individuals detected at carcasses (individual-based rarefaction) and the y-axis shows the effective number of species for three diversity orders: q = 0 (species richness, panels a and b), q = 1 (species evenness, panels c and d), and q = 2 (species dominance, panels e and f). Solid lines represent rarefaction (interpolation) based on observed data, and dashed lines represent extrapolation beyond the observed sample size. Within each plot, each line represents a sampling site, illustrating how diversity accumulates with sampling effort.

Species composition and environmental correlates of vertebrates using carrion. (a) Heat map showing species observed using carrion at each carcass. The x-axis represents carcass grouped by sampling location, and the y-axis lists species. Each cell indicates the relative abundance of a species at a given carcass; dotted lines delimit sampling locations. (b) Redundancy analysis (RDA) biplot showing relationships between environmental variables and species composition across carcasses (n = 70). Points represent individual carcasses, coloured according to livestock pressure, and shaped according to province. Arrows indicate the direction and strength of environmental predictors, and proximity between points denotes similarity in species composition.
RDA explained 49.1% of compositional variance (global F = 7.35, p < 0.001; Fig. 3b). The first three axes (RDA1 = 27.5%, RDA2 = 10.6%, RDA3 = 5.8%) jointly explained 43.9% (p < 0.001). Province, livestock management pressure, initial carcass mass, vegetation cover, and the province-by-pressure were significant (p ≤ 0.047), whereas carcass duration was not (p = 0.273). RDA1 separated provinces; RDA2 captured the pressure gradient. Pairwise PERMANOVA confirmed differences between no- and high-pressure (p = 0.001) and between no- vs medium-pressure (p = 0.002) sites, with high vs medium marginal (p = 0.057).
For richness (q = 0), both presence- and abundance-based analyses most often supported the hierarchy model (H7, 59.2% and 35.6% of bootstraps). Puma, culpeo fox, and Andean condor were key predictors (importance > 0.70). In presence data (Fig. 4a), all had positive effects: puma 45% (exp β = 1.45; 95% CI = 1.17–1.97), culpeo fox 36% (1.36, 1.15–1.59), Andean condor 27% (1.27, 1.07–1.46). No-pressure sites showed 27% lower richness vs high-pressure (0.73; 95%, 0.56−0.98). In abundance data (Fig. 4b), Andean condor (2%, 1.02, 1.00–1.03) and culpeo fox (14%, 1.14, 1.01–1.27) were positive; puma was positive but not significant.

Multiplicative effects of ecological predictors on the diversity of vertebrates using carrion across Hill numbers: (a, b) species richness (q = 0), (c, d) evenness (q = 1), and (e, f) dominance (q = 2). Left panels show presence-based models, right panels abundance-based models. Diamonds indicate model-averaged coefficients (500 bootstrap iterations); thick and thin bars represent 90% and 95% percentile confidence intervals, respectively. Diamond colours denote variable importance, calculated as the sum of Akaike weights across the supported model set. Predictors include dominant scavengers (Andean condor, grey fox, kelp gull), large apex carnivores (puma, culpeo fox), and environmental variables (livestock management pressure, vegetation cover, carcass mass, carcass duration). Livestock management pressure was treated as categorical (baseline = high pressure).
For q = 1, presence data most strongly supported the environment + apex hypothesis (H8, 55.4%). Puma and culpeo fox presence increased diversity by 45% (1.45, 1.14–1.93) and 29% (1.29, 1.09–1.51), respectively, while medium pressure reduced it by ∼19% (0.81, 0.69−0.95; Fig. 4c). In abundance data (Fig. 4d), support was diffuse; the dominant model (H6, 23.8%) led, with grey fox abundance showing a negative effect (-7.5%, 0.93, 0.86−0.98).
For q = 2, presence data again supported H8 (37.8%), with puma increasing diversity by 41% (1.41, 1.08–2.14). Medium pressure reduced it by 24% (0.76, 0.62−0.92). In abundance data (Fig. 4f), the full model (H10, 37.8%) prevailed; only Andean condor abundance was significant, decreasing diversity by 2.7% on average (0.97, 0.96−0.99).
Large carnivore presence (puma and culpeo fox) was positively associated with richness and evenness of vertebrates using carrion (q = 0, 1). In contrast, higher relative abundance of grey fox was associated with lower evenness (q = 1), and Andean condor abundance showed a weak negative association with higher-order diversity (q = 2). Livestock management pressure was also associated with diversity patterns, although effects were detected primarily in presence-based models. The best-supported richness model (H7) included puma, culpeo fox, and Andean condor as positive predictors of richness, indicating that multiple species identities were associated with variation in the diversity of vertebrates using carrion among carcasses.
DiscussionOur results show that vertebrate scavenger guild assembly in the Patagonian steppe is structured by interacting patterns consistent with facilitation, dominance, and environmental filtering, producing a multidimensional and non-additive community structure. By examining carcass assemblages along a livestock management pressure gradient, we identified how species traits and management regimes are associated with variation in scavenger diversity.
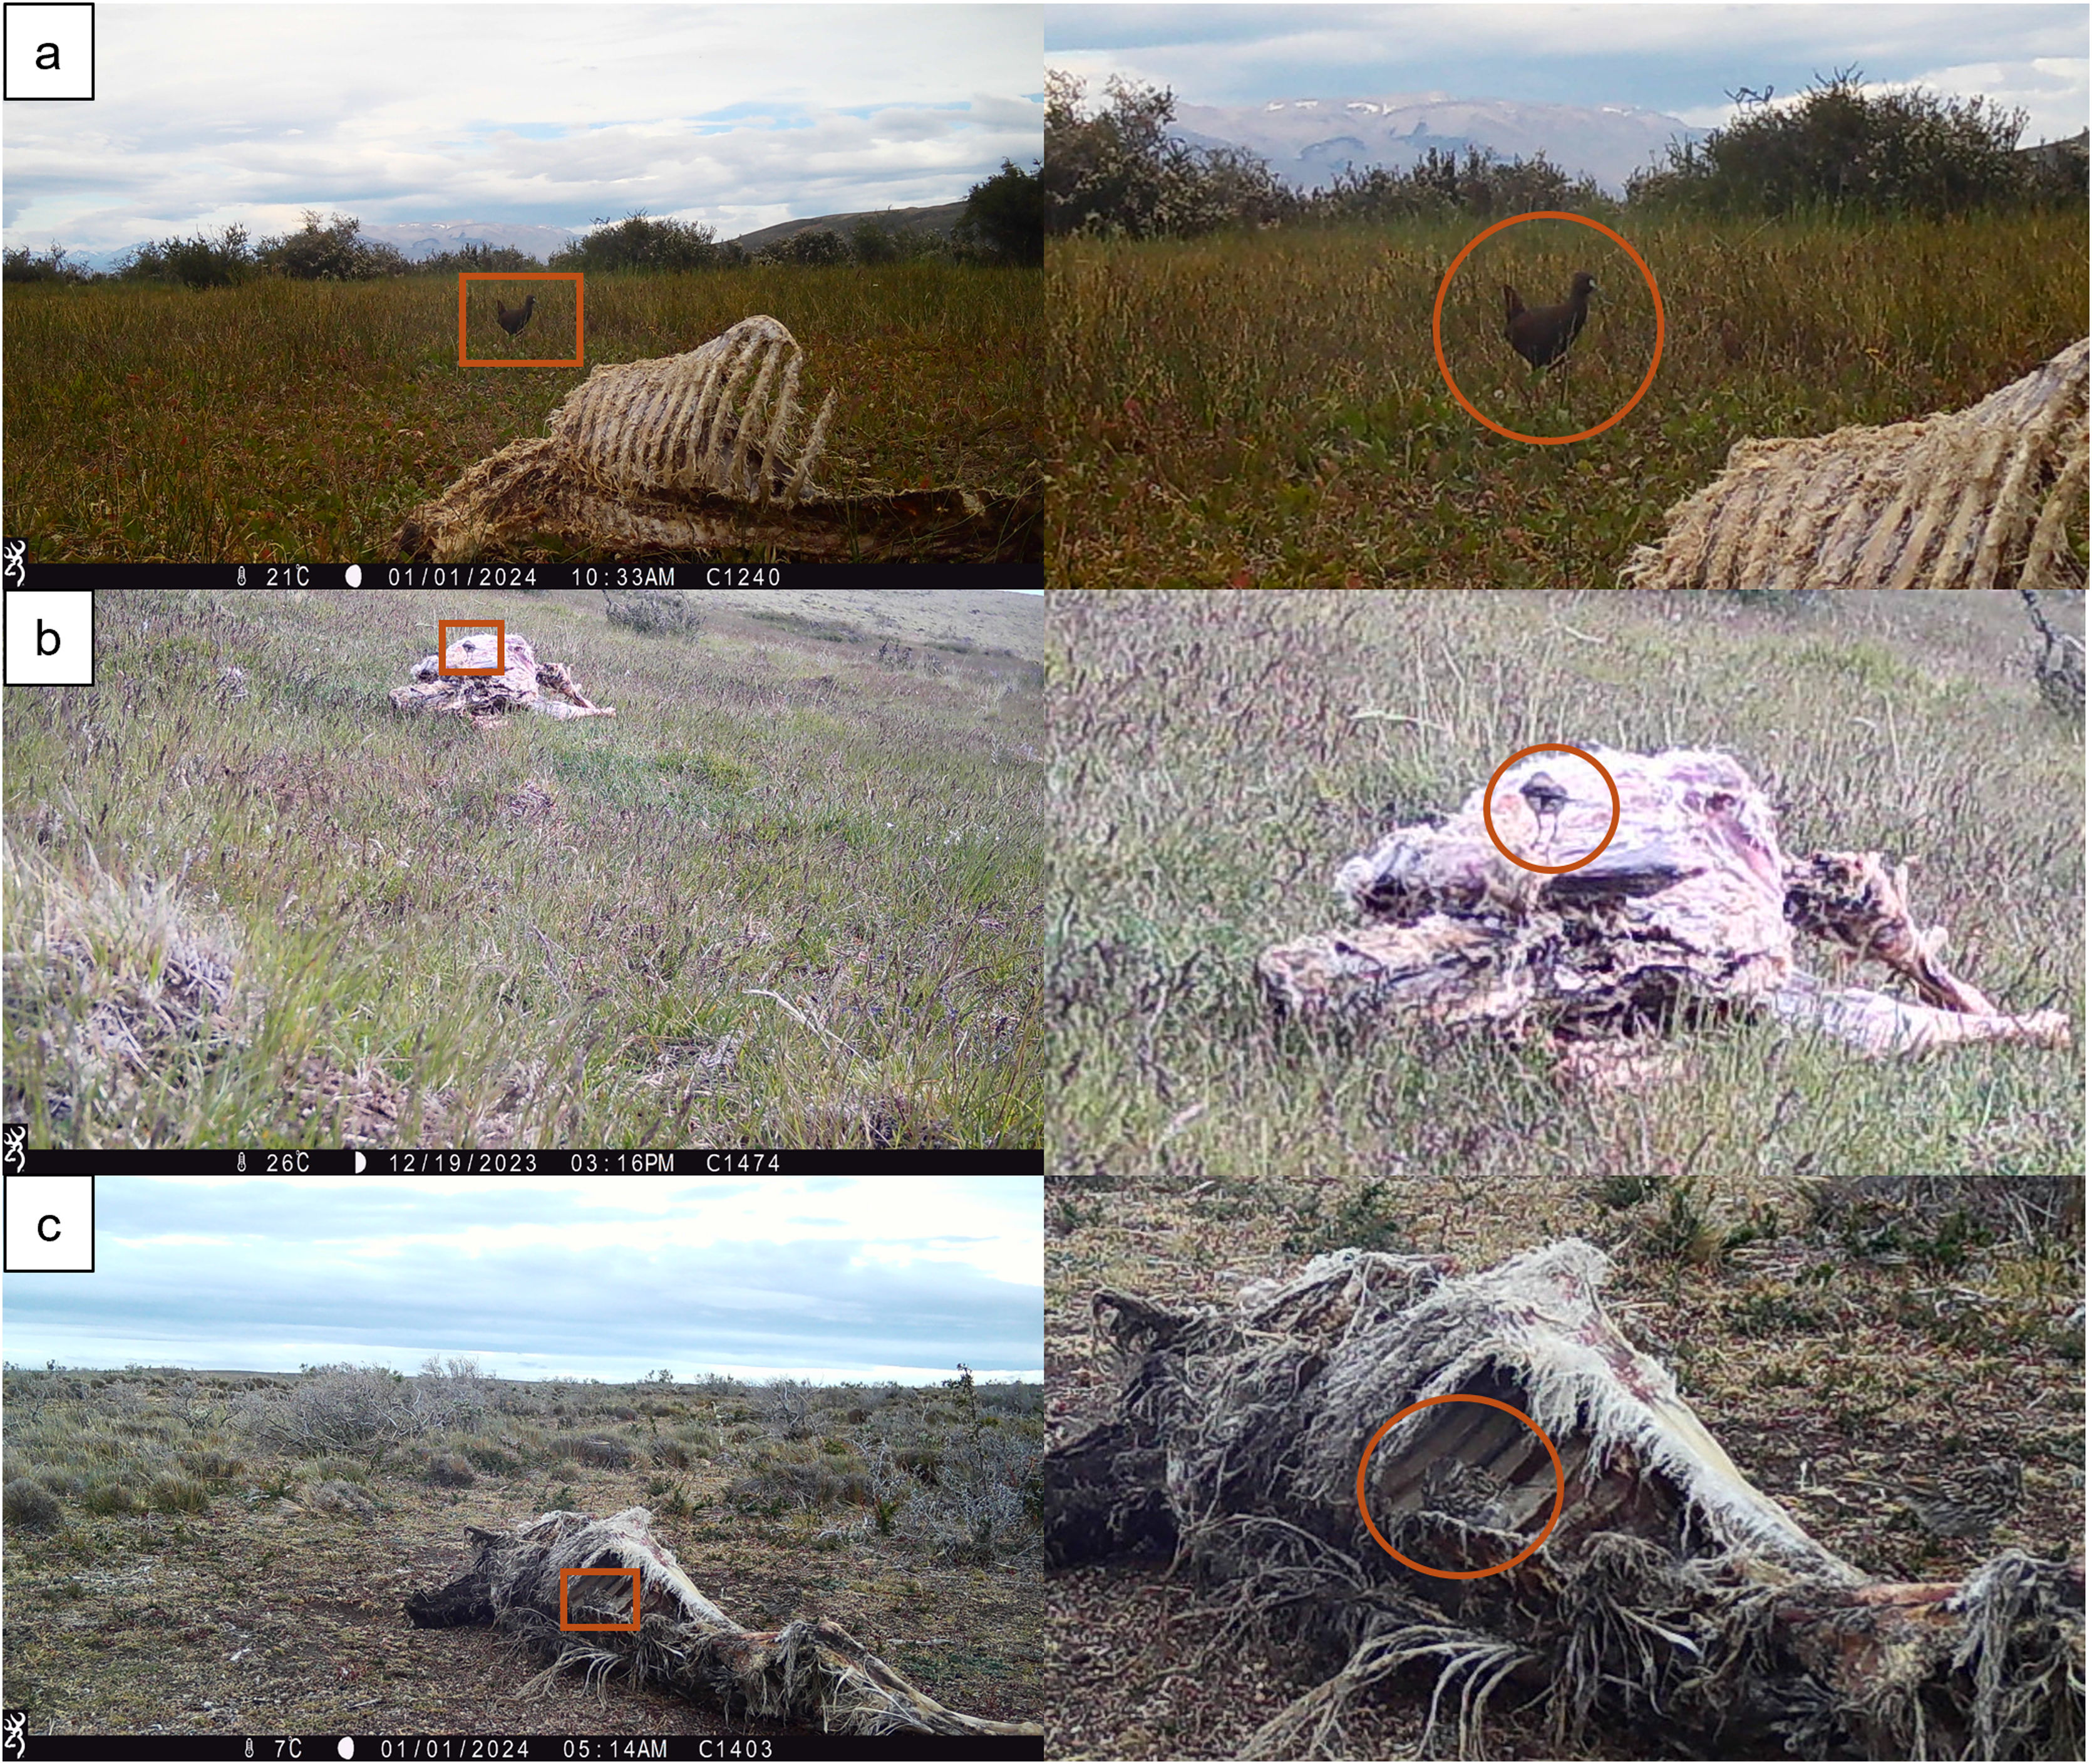
We recorded 41 vertebrate species using carrion, including 16 species observed directly consuming carcass tissues and 25 species exhibiting fluid consumption or undetermined use. The overall richness of carrion-associated vertebrates represents the highest value reported for any steppe ecosystem. Among direct carrion consumers alone, richness remained exceptionally high compared with values reported across 2,485 carcasses in 43 global studies (Sebastián-González et al., 2019) and surpasses values from species-rich systems such as the Brazilian Cerrado (n = 19; Naves-Alegre et al., 2021), Californian forests (29; Allen et al., 2014), and temperate forests in eastern Europe (≤36; Selva et al., 2005). It also contrasts with the Mongolian Gobi (8) and previous studies from Patagonia (5–9, Orihuela-Torres et al., 2021). The broader estimate of 41 species further highlights that carrion can support a wider assemblage of vertebrates beyond direct tissue consumers. Such richness is notable given Patagonia’s harsh abiotic conditions –low temperatures, strong winds, and sparse vegetation (Radic-Schilling et al., 2024; Waide et al., 1999).
Under these constraints, carrion functions as a spatially scattered subsidy that attracts a broad array of consumers (DeVault et al., 2003). Our models indicate that functional roles and livestock-related factors, rather than background environmental harshness, were more strongly associated with community structure. Extensive ranching may increase carrion availability, potentially sustaining diverse scavenger assemblages (Olea and Mateo-Tomás, 2009; Oro et al., 2013).
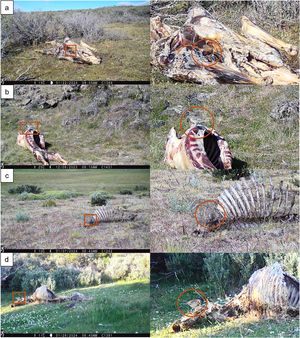
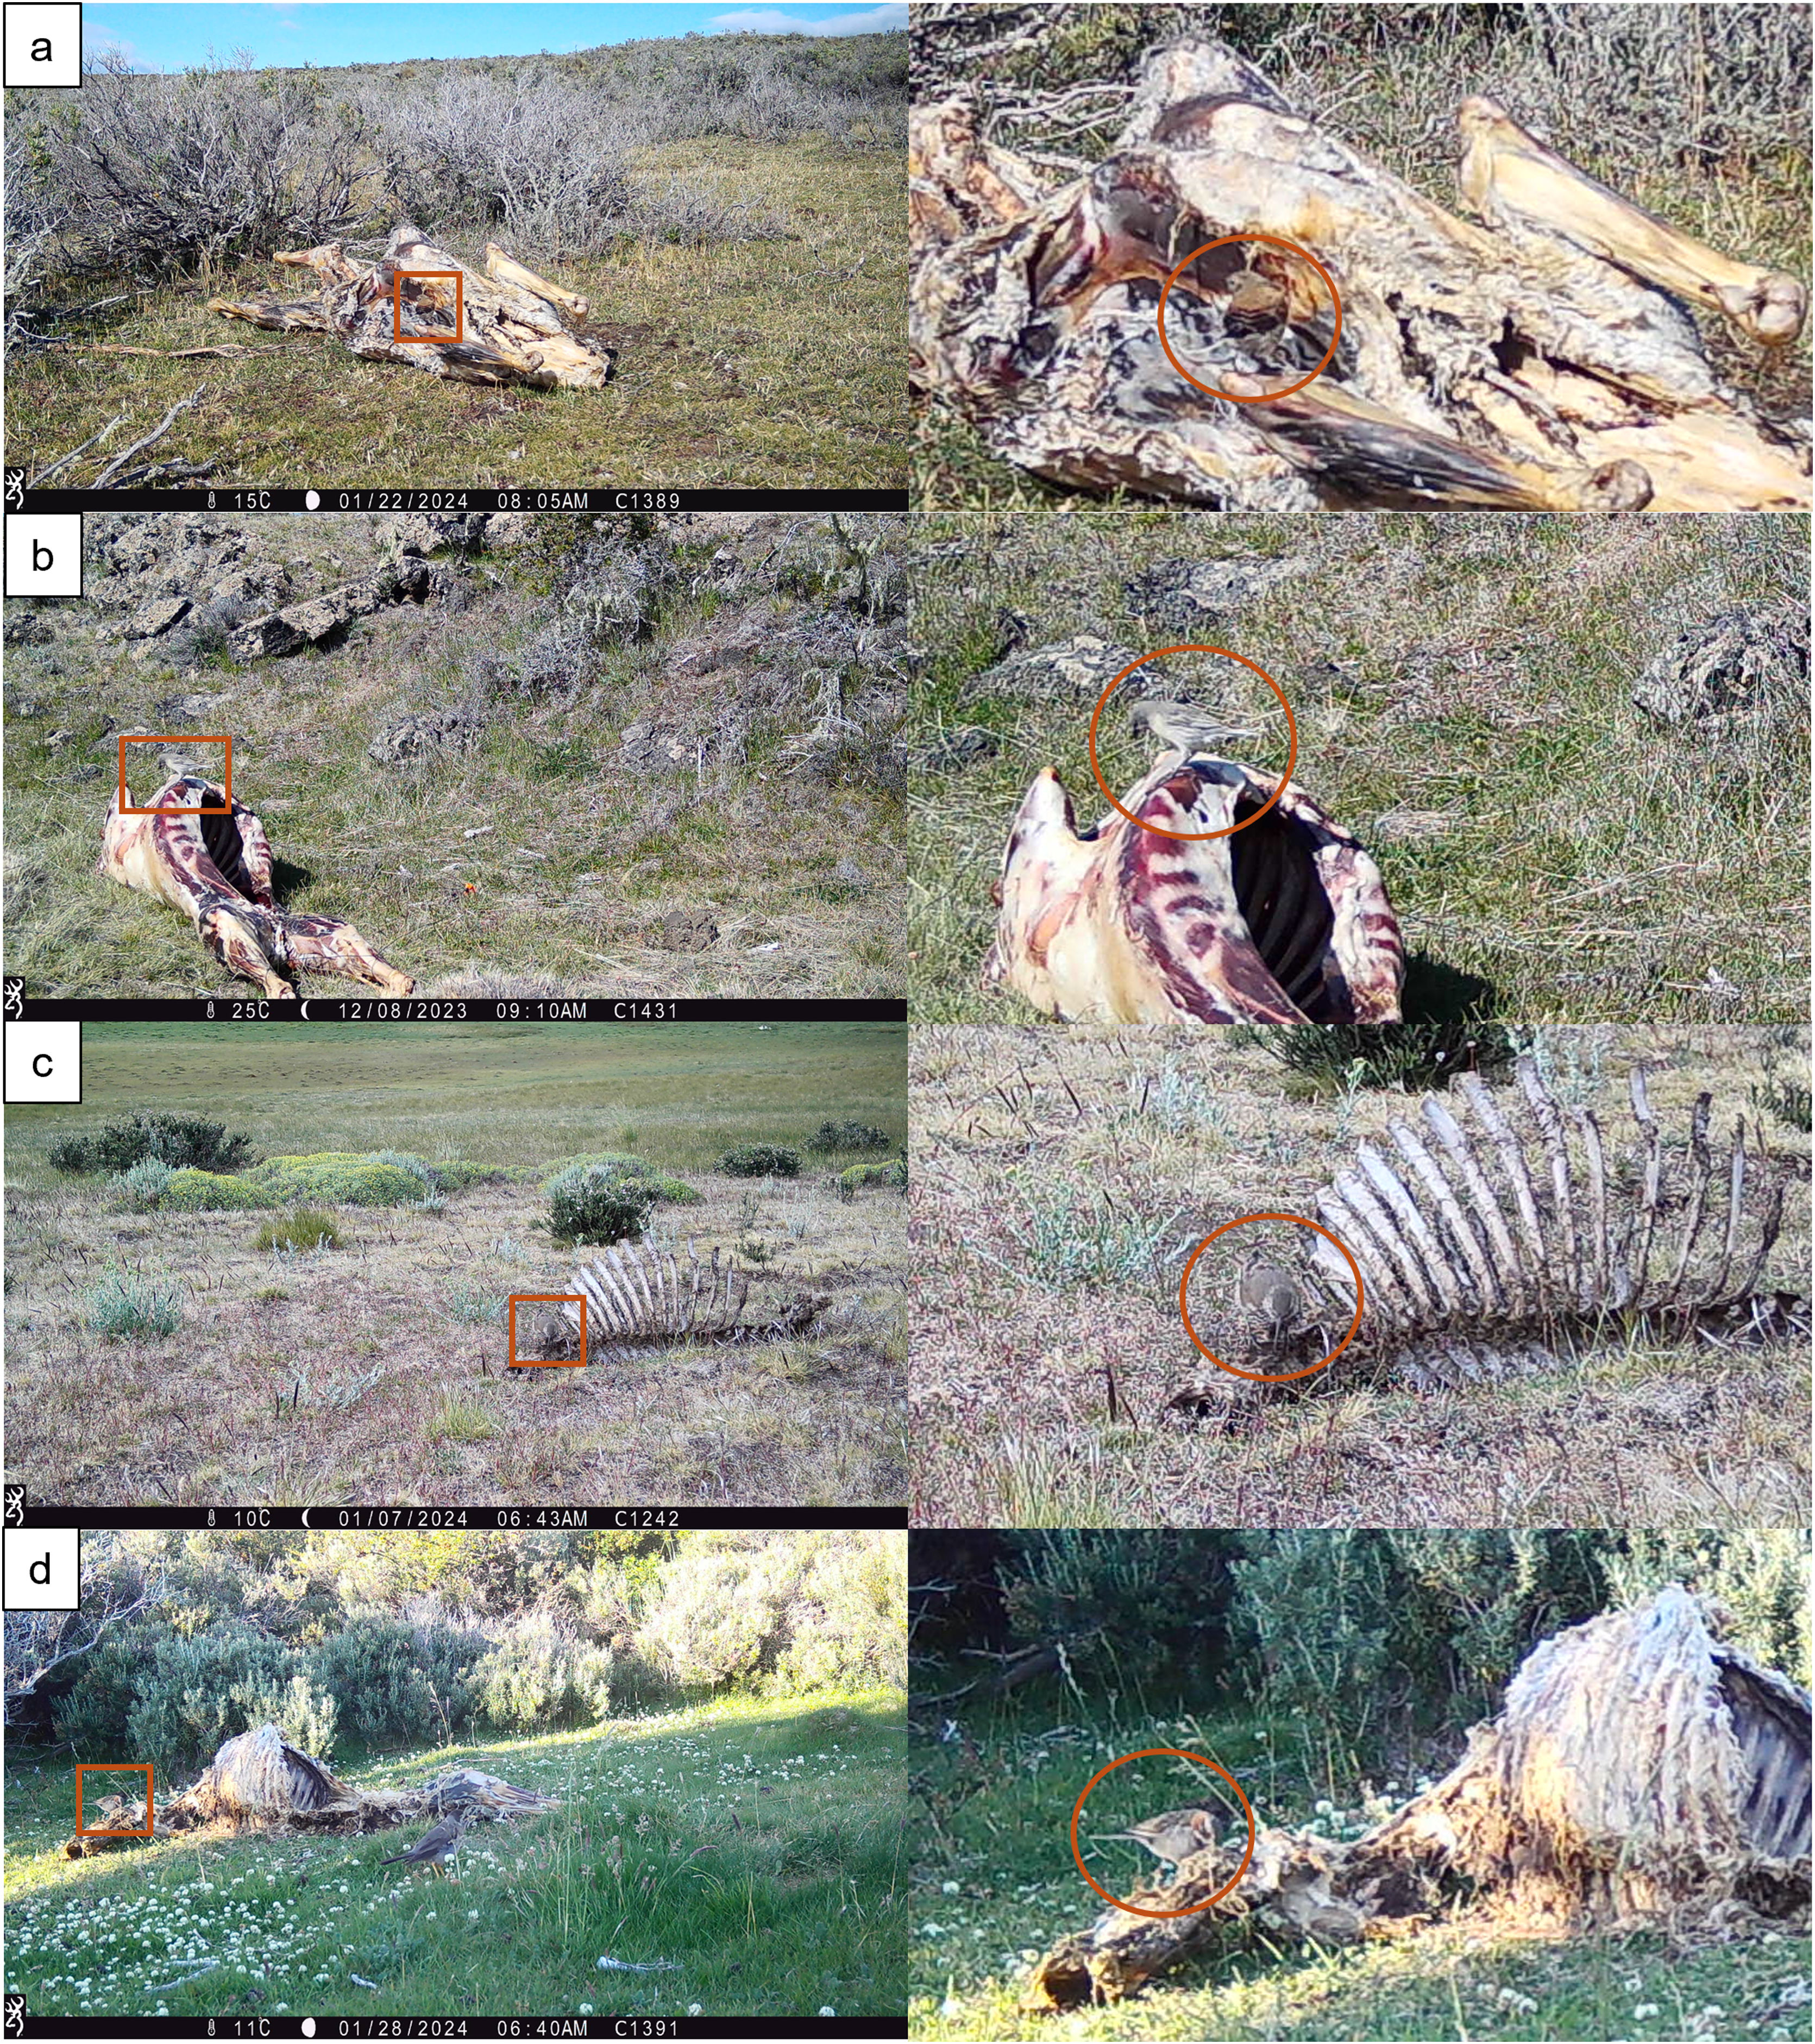
Large apex carnivores (puma and culpeo fox) were consistently associated with higher richness and evenness. These patterns are compatible with facilitative mechanisms, such as behavioural modulation or temporal niche segregation (Allen et al., 2014), although alternative explanations—including shared habitat preferences, baseline differences in carrion availability, or unmeasured environmental factors such as topographic ruggedness, prey density, or proximity to refuges—cannot be excluded. Nevertheless, the consistent positive association between large carnivore presence and evenness across sites, even after accounting for measured environmental variables, suggests that biotic interactions may contribute to these patterns. Moreover, we documented > 20 passerines using carcasses –taxa seldom classified as scavengers– suggesting that carrion use by small vertebrates may be underestimated in open ecosystems.
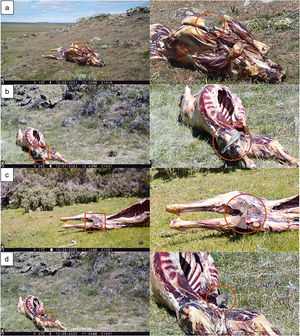
Although some passerines may consume insects associated with carrion rather than vertebrate tissue, such interactions still represent trophic use of carcass-associated resources. Previous syntheses highlight that carrion exploitation by vertebrates has likely been underestimated due to narrow dietary classifications (DeVault et al., 2003). Passerine use of carcasses—including pecking of soft tissues and fluid intake—has been documented in multiple systems (Moreno-Opo and Margalida, 2013). Similar observations have been reported in other systems, where passerines are frequently recorded at carcasses, although their specific feeding behaviour (e.g., tissue vs. invertebrate consumption) is not always clearly distinguished (Elbroch et al., 2017). Likewise, occasional necrophagy by nominally herbivorous mammals has been reported, particularly involving ingestion of soft tissues or bodily fluids, indicating that occasional carrion consumption is not limited to taxa traditionally classified as scavengers (Wenting et al., 2022). In our study, carrion use was restricted to visible direct interaction with carcass tissue or fluids, minimizing the risk of overestimating scavenging events.
Scavenger composition varied markedly between provinces and sites. Although province was a significant compositional axis in the RDA, it lost predictive power for Hill-number diversity once large carnivore presence, dominance, and livestock management pressure were considered. Landscape structure may modulate these effects (Pardo-Barquín et al., 2019), the rugged topography ULT versus the flat terrain of MAG (Radic-Schilling et al., 2024) may explain why Andean condor numerically dominated carcasses only in the former, where wind and relief facilitate soaring and access to carcasses. Similar spatial segregation of raptors occurs in Mongolian steppe system, where raptors are associated with mountainous areas offering shelter, climatic buffering, and nesting or roosting sites (Orihuela-Torres et al., 2021).
Consumer identity was strongly associated with guild structure (Tobajas et al., 2021; Mateo-Tomás et al., 2017). This pattern is consistent with interaction-based frameworks recognizing that species differ in their ecological roles within scavenger assemblages depending on trophic position and their influence on access to carrion resources (Inagaki et al., 2025). In our study, carcasses where large carnivores were present tended to exhibit higher evenness, whereas assemblages numerically dominated by a single species were characterized by lower evenness values. While these patterns are consistent with behavioural modulation or temporal segregation among consumers (Bell et al., 2023), they remain correlational. Interestingly, the absence of obligate scavengers (e.g., Andean condor) did not necessarily coincide with lower diversity, as facultative species were more prevalent at some carcasses. However, numerical compensation does not necessarily imply functional equivalence, particularly if substitute taxa differ in carcass detection efficiency, processing capacity, or spatial mobility (Hill et al., 2018; Olson et al., 2012). For example, large obligate scavengers such as the Andean condor can substantially accelerate carcass consumption and removal due to their high detection efficiency and feeding capacity (Méndez et al., 2024).
Two caveats merit mention. First, facilitation mechanisms are inferred from richness and evenness patterns, and our analyses are correlational. Behavioural interactions and carcass removal rates were not directly quantified; experimental or fine-scale temporal data would be required to establish causality (Syme et al., 2024). Second, livestock management pressure effects appeared mainly in presence-based models, suggesting that filters may operate primarily on occurrence rather than abundance; future work should separate arrival and persistence processes and include detection correction (Fern et al., 2020).
Implications for conservation and managementPrevious studies have highlighted the ecological importance of large carnivores in structuring scavenger assemblages (Allen et al., 2015; Ordiz et al., 2013). In our system, large apex carnivores were positively associated with carcass-level richness and evenness, suggesting that maintaining viable populations may contribute to sustaining diversity patterns. Likewise, understanding conditions under which certain species numerically dominate carcasses may help anticipate shifts in assemblage structure (Rees et al., 2024). Because carcass removal rates and functional efficiency were not directly quantified, these implications should be interpreted cautiously. The sensitivity of occurrence-level diversity to livestock management pressure suggests that moderating persecution and promoting habitat heterogeneity could help buffer scavenger communities against compositional shifts. Further behavioural and experimental work is needed to clarify how variation in guild structure translates into ecosystem functioning in landscapes increasingly shaped by human activity.
CRediT authorship contribution statementM.J.-T., M.R.-A., and P.C. conceived the ideas and designed the methodology. M.R.-A., R.H., S.R.-S., and P.C. collected the data. M.J.-T., M.R.-A., and P.C. analysed and interpreted the data. M.J.-T., and P.C. led the writing of the manuscript. All authors contributed critically to the drafts and gave final approval for publication.
Declaration of Generative AI and AI-assisted technologies in the writing processThe authors used ChatGPT 5.0 to identify and correct grammar, spelling, and stylistic issues in the manuscript, and to help with R coding. All content was subsequently reviewed and edited by the authors, who take full responsibility for the final published version.
FundingThis research was supported by ANID-Chile through FONDECYT Regular project 1230422 awarded to P. Corti and S. Radic-Schilling. M. Jiménez-Torres received support from ANID-Subdirección de Capital Humano/Doctorado Nacional/2022-21221530. M. Ruiz-Aravena was supported by the U.S. Forest Service International Programs (Agreement 22-DG-11132762-347), as part of his contribution to the Forest and Wildlife Research Center, Mississippi State University. This work also received funding from McIntire-Stennis. The funders had no role in study design, data collection and analysis, manuscript preparation, or the decision to submit the article for publication.
Data availabilityData will be available upon completion of the study, except for components withheld to protect the privacy of ranch owners.
The authors declare no competing interests.
We thank the Chilean Forest Service (CONAF) at Magallanes District for authorizing access to National Parks. Cerro Guido Foundation and Ranching, La Portada and Josefina ranches, for granting land access and logistical support. We also acknowledge the Municipality of Torres del Paine and Centro IDeAL for providing lodging facilities. We thank N. Diez, J. Cabezas, and G. Biscarra for assisting with the identification of passerine species. A. Martin, F. Arce, and M. Vega for fieldwork assistance. We also acknowledge PECON for making available a free open-access platform dedicated to fostering rigorous ecology-conservation science across Latin American countries.