

Several studies have highlighted the impacts of roads and highways on species dispersal, abundance, and persistence, since these are the infrastructures that most threaten biodiversity. Yet, little is known about how roads affect community assembly processes at broader spatial extents. Understanding interactions between roads and community assembly processes is an urgent need especially in tropical areas, where key biodiversity hotspots and ecosystem services are critically threatened. Here, we review how roads could shape community assembly processes and (meta)community structure across biogeographic extents for animals, with a focus on identifying causal effects. We use causal diagrams to illustrate the expected relationships among variables representing processes influencing species composition and dissimilarity under road influence. In doing so, we highlight how observational studies on road effects are prone to confounding and bias, using the concrete example of the controversial BR-319 highway in the Amazon. We propose the use of quasi-experimental designs as an alternative for better assessing the impacts of roads’ construction on animal communities. We conclude that more integrated and multi-process approaches are needed to study (meta)communities, moving from mere descriptions of correlations to the identification of the causality of ecological processes. This can be more easily achieved by integrating spatial and temporal ecological data.

Roads and highways are considered the human infrastructures that most threaten terrestrial ecosystems and biodiversity (IUCN, 2023). For about 30 years, highways have received special attention from ecology researchers who seek to understand the interactions among biodiversity, landscape and human infrastructures. From that, literature reviews have highlighted the mostly negative impacts of roads on species dispersal, abundance, and persistence (Forman and Alexander, 1998; Coffin, 2007; Shepard et al., 2008; Balkenhol and Waits, 2009; Fensome and Mathews, 2016). Furthermore, roads may play new roles for many species as their ranges shift under anthropogenic modification of their habitats (Caplat et al., 2016).
Correlations between highways and local wildlife are widely known. Two major effects have emerged, the “edge effect” and the “barrier effect”. The edge effect is typically identified as a correlation between some aspects of biodiversity or ecosystem and the perpendicular distance to a road. These effects may arise from the direct mortality of individuals due to roadkill, which can reduce local abundance or alter community composition near the road edge, but also from indirect habitat-related impacts, such as noise, chemical pollution, and other forms of habitat degradation (Da Rosa and Bager, 2013). The barrier effect is an increase in dissimilarity between roadsides in any aspect of biodiversity, presumably due to dispersal limitation. For instance, roadkill, one of the main impacts on terrestrial wildlife, could work as a filter that modifies the patterns of displacement and genetic exchange of biological populations living near roads. While the barrier effect is mainly observed in low mobility species, such as small mammals and forest specialist birds, roads can even serve as displacement corridors for medium and large mammals (Fahrig e Rytwinski, 2009). Both the edge and barrier effect could affect community assembly processes occurring across communities influenced by the road. On the other hand, dispersal could connect local communities that thereby could function as metacommunities (Hubbell, 2001; Vellend, 2016; Leibold and Chase, 2018).
There are two major uncertainties in these expectations. First, much of the literature on road biodiversity effects is based on correlations measured on observational data. Therefore, there is much potential for bias being introduced by unknown and/or unmeasured confounders (Shipley, 2016; Arif and MacNeil, 2022; Tan and Zhou, 2023). Second, little is known about how road effects act at the metacommunity level (i.e. sets of communities connected by dispersal on different parts of the road), which becomes an important knowledge gap for biodiversity conservation, since many roads traverse hundreds or thousands of kilometers (Laurance et al., 2009). Understanding how strategic roads affect the ecology of communities is important because the effects of local ecological processes can interact with dispersal and with each other over larger spatial extents (Siqueira et al., 2020; Jacobi and Siqueira, 2023) or may even be overridden by dispersal effects. Such variation could modify the impact of a road on all metacommunities along the road. Yet interactions among ecological processes have received mainly theoretical attention so far, and the potential for anthropogenic mediation of such interactions (e.g. by human structures such as roads) is unclear.
Understanding interactions between roads and metacommunity processes is an urgent need in tropical areas, where key biodiversity hotspots and ecosystem services are critically threatened by human activities (Levis et al., 2020). Tropical forests are traversed by roads and highways across the world, such as the Andaman Trunk Road in India (420 km), the Douala–Bangui Road in the African Congo Basin (1400 km), and the Belém–Brasília Highway in Brazilian Amazonia (2000 km) (Laurance et al., 2009). These roads have largely promoted deforestation by facilitating human access and the consequent expansion of logging, mining, agriculture, hunting, and wildfires (Laurance et al., 2009; Alamgir et al., 2017; Kleinschroth and Healey, 2017). Further, over 20 million km of paved roads are expected to be built or paved by 2050 in developing countries, most of which are in the tropics (Alamgir et al., 2017). A typical example is the 80 km long non-paved road PR-405 that connects Antonina to Guaraqueçaba municipalities in the greatest remnant of Atlantic Forest (Silva et al., 2007). The access by water or by a dirty road, associated with private and public protected areas, are the main factors contributing to the conservation of this area and so the biome. However, even narrow, unpaved roads with low traffic and speed can be avoided by some species, thus possibly limiting dispersal even in the absence of roadkill (Goosem, 2001). Tropical forest specialists typically avoid forest edges and, thus, road clearings (Laurance et al., 2009).
Here, we elaborate on how roads could shape community assembly processes and (meta)community structure across biogeographic extents (i.e. hundreds of kilometers) for animals. Specifically, we use causal diagrams (i.e. Directed Acyclic Graphs; Shipley, 2016) to clarify how roads may shape community assembly processes, to highlight how observational studies on road effects are prone to confounding and bias, and to motivate sampling designs that might allow causal identification of road effects. We will focus on species composition and its dissimilarity between communities, as these features have proved most informative about community assembly processes and metacommunity structure (Tuomisto and Ruokolainen, 2006; Vellend, 2016; Soininen, 2014; Leibold and Chase, 2018). We consider three response variables at different spatial scales which are typically used to investigate community assembly: (1) the species composition of a local community at some geographic position within the zone of influence along the road; (2) the compositional dissimilarity between a pair of local communities, either on the same side or on opposite sides of the road (pairwise beta diversity); and (3) the total dissimilarity of a metacommunity (set of local communities) in some section of the road, either adjacent to or traversed by the road. We use a concrete example to illustrate the challenges and opportunities in estimating road effects on (meta)communities: the BR-319, an 885 km long road in Brazilian Amazonia built in the 1970s whose regular use has been discontinued since the 1980s, but whose asphalt pavement installation has been receiving strong political and popular support.
Community assembly processes and species composition and dissimilarityA contemporary view of the reason why the composition of local communities vary can be summarized in four higher-level processes: natural selection, ecological drift, dispersal and speciation (Hubbell, 2001; Hanson et al., 2012; Vellend, 2010, 2016; Leibold and Chase, 2018). Natural selection, or environmental selection (Vellend, 2010), is the process by which certain individuals are favored over others based on their adaptive characteristics to the abiotic or biotic environment (Darwin, 1859). As species differ in their traits, selection should also favor certain species over others depending on environmental conditions, also known as “species sorting” or “environmental filtering” (Hanson et al., 2012; Vellend, 2016; Leibold and Chase, 2018). Accordingly, the composition of local communities should be correlated with environmental conditions, and compositional dissimilarity should increase with environmental distance along the filtering variable.
Yet, variation in species composition does not require environmental variation. Ecological drift refers to random changes in the composition of species in a community (Hubbell, 2001). This occurs because the contribution of individuals to the next generation is variable: not all individuals survive or reproduce equally. This implies that, all else being equal, the next generation of species in a community will represent a sample of the current generation, being subject to sampling error – which in this context is typically called “demographic stochasticity” (Hubbell, 2001). Consequently, over time, species can become locally extinct by chance, and this chance increases with increasing time and decreasing population size, when sampling error becomes stronger (Hubbell, 2001). Therefore, under the sole effect of ecological drift, the composition of a local community should change randomly over time due to random species extinctions, and the rate of random species loss should increase as community size (or total number of individuals) decreases. Likewise, the compositional dissimilarity among a set of communities (metacommunity) should increase over time, and more so in metacommunities with lower mean community size. Furthermore, differences in species composition should be weaklier related to environmental differences in metacommunities with lower mean community size, as random extinctions should dilute the nonrandom effect of selection (Siqueira et al., 2020).
Dispersal is the movement of individuals between different places (Hubbell, 2001; Hanson et al., 2012; Vellend, 2016; Leibold and Chase, 2018). In general, we can expect dispersal rates between communities to decrease with increasing geographic distance and with the occurrence of dispersal barriers between sites, either natural barriers such as mountains and rivers or anthropogenic barriers such as cities and roads. Therefore, local species composition should change as a function of distance to the nearest source of colonizers, while compositional dissimilarity should increase with increasing geographic distance between communities (Hubbell, 2001; Hanson et al., 2012; Vellend, 2016; Leibold and Chase, 2018). Moreover, communities on opposite sides of a dispersal barrier (e.g. river or road) should have greater composition dissimilarity than communities on the same side of the barrier. At the metacommunity level, a dispersal barrier traversing the metacommunity should increase overall compositional dissimilarity, and this effect should be stronger where mean community size is smaller due to the stronger ecological drift (Hubbell, 2001; Hanson et al., 2012; Vellend, 2016).
Speciation is the divergence of ancestral species into new species (see Shapiro et al., 2016 for a conceptual review). Such divergence results from evolution of reproductive isolation between populations, which tends to increase as populations accumulate genetic differences (Mallet, 2008). As such, speciation may be driven by geographic insulation (e.g. due to dispersal limitation and genetic drift), divergent selection (e.g. due to contrasting habitats), or both. Likewise, a population may diverge locally due to divergent selection, as in sympatric speciation, or between non-overlapping areas where dispersal limitation and genetic drift are likely to be as or more important than selection (e.g. parapatric or allopatric speciation) (Rosser et al., 2015). Speciation may be considered negligible under the time span considered by most ecological studies and will not be further considered here. However, speciation is clearly required for the maintenance of biodiversity in the long term (Hubbell, 2001; Vellend, 2016), historical patterns of speciation may still shape current metacommunity patterns (Vellend, 2016), and incomplete or ongoing speciation may also be relevant in a community context as diverging population may differ in their environmental responses (Shafer and Wolf, 2013).
Overall, selection and ecological drift eliminate species from local communities (by impairing their persistence based on their traits or by chance, respectively) and thus tend to increase the compositional dissimilarity within metacommunities. In contrast, dispersal adds species to local communities by exchanging them among sites and thus tends to decrease the compositional dissimilarity within metacommunities. Furthermore, the relative importance of each mentioned process should depend on the spatial and temporal scale (i.e. size of local communities) and extent (i.e. total area or time span covered by local communities) (Leibold and Chase, 2018; Lu and Jetz, 2023; Shinohara et al., 2023) and the interaction between them (Fodelianakis et al., 2021; Mendoza et al., 2015). Specifically, we may expect dispersal limitation to increase with increasing spatial extent due to larger geographic distances and increased likelihood that geographic barriers will be encompassed by the area. Likewise, we may expect stronger selection and wider abundance gradients (which underlie the strength of ecological drift) as environmental heterogeneity increases, and the latter is also likely to increase with spatial extent. Consequently, we may also expect stronger interaction between ecological processes with increasing spatial extent. It is this latter aspect that may be particularly important in the context of roads traversing large distances and several habitat types, such as many roads in tropical forests.
What is a road (meta)community?The definition of a metacommunity is arbitrary, depending primarily on the issue under analysis and the dispersal capacity of the taxon. However, defining a metacommunity on a scale that encompasses the entire length of a road is informative when the goal is to understand the effect of large tropical highways that traverse large-scale environmental gradients.Thus, we define our sampling universe as the entire road metacommunity: the set of local communities within the total area of influence along a road. In turn, a local community is defined as the set of species and their individuals of a given taxon occurring together within a site much smaller than the total area of the road metacommunity. We can approximate the physical limits of the road metacommunity by considering the maximum distance of its edge effect. While this distance varies depending on the variable or organism considered, edge effects can occur up to several kilometers in tropical forests due to wildfires, a major driver of deforestation and forest degradation (Laurance, 2000; Cochrane and Laurance, 2002; Lapola et al., 2023; Flores et al., 2024). For instance, in Amazonia, 50% of satellite wildfire detections occur within 1 km from any road or river, but 95% occur within 10 km (Kumar et al., 2014; Armenteras et al., 2017). Therefore, assuming a 10-km influence zone on each roadside, a 1000-km long road (which is within the range of large roads traversing tropical forests worldwide) would encompass around 20.000 km². Within this area, we could place 2 million 1-ha plots, the typical scale used to sample tree communities in tropical forests (Lima et al., 2023). This whole area is similar to that of entire countries such as El Salvador, Israel, or Wales, which helps one to envision the potential extent of road effects.
Road edge effects on community compositionEdge effects are typically inferred from a correlation between some aspects of biodiversity (e.g. species composition, as represented by an ordination score) at a given site and its perpendicular distance to an edge (Goosem, 2001; Ruffell and Didham, 2016; Ries et al., 2017). This correlation is often nonlinear and can be thought of as having two components: the “depth” or maximum distance to which the edge has an effect; and the “magnitude”, or degree of difference between communities near vs. away from the edge (Ries et al., 2017). In the case of roads, edge effects could be either direct or indirect. The major direct effect of roads on species is mortality caused by roadkill (Forman and Alexander, 1998; Shepard et al., 2008; Ceia-Hasse et al., 2018). If species vary in their probability of dispersing across the road and/or dying during the process, the road creates source-sink dynamics between sites farther (sources) and closer (sinks) to the road, changing species composition near the road regardless of the environment. The major indirect effect is: roads are the main agents of habitat loss, by increasing habitat fragmentation, ecosystem isolation and modification of the local environmental conditions on roadsides such as soil, vegetation and microclimate, and create modified landscapes and gradients of environmental pollution (Forman and Alexander, 1998; Shepard et al., 2008; Ceia-Hasse et al., 2018). Likewise, roads increase accessibility by humans, promoting other sources of wildlife mortality such as hunting (Laurance et al., 2009). The implementation of roads, mainly paved ones, also increases selective logging, wildfire events and spread of important diseases such as malaria (Nepstad et al., 2001; Espinosa et al., 2014; Hethcoat et al., 2020; Hahn et al., 2014). In fact, most edge effects are thought to be indirect, through changes in the distribution of resources and/or abiotic conditions that affect species differently (Ruffell and Didham, 2016; Ries et al., 2017). Beyond this, intensity of use (e.g. traffic rate) can vary along the road and may influence the edge effect itself, e.g. if direct mortality is higher or environmental conditions near the road are more strongly modified in more intensively used road sections. If so, local species composition should respond to a statistical interaction between distance from road and road use intensity.
Despite these predictions, there are at least two issues that complicate interpreting correlations between species composition and road distance as caused by roads. First, species composition can respond to the environment independently of the road, e.g. environmental gradients that already existed before the road. In fact, pre-existing environmental gradients can themselves affect distance to the road, as road engineers often consider environmental features (e.g. topography, flood risk) to determine road position (Subramani and Pari, 2015). Second, local communities can differ in species composition through dispersal limitations simply by being in different geographic positions, regardless of environment. In nature, distance from the road and geographic position are necessarily correlated, and both can correlate with pre-existing environmental gradients due to spatial autocorrelation in the environment. Therefore, any correlation between species composition and distance from road potentially confounds edge effects (both direct and indirect) with environmental and spatial effects (Fig. 1).

Causal diagram showing expected relationships between species composition, distance from road, environment, and geography across local communities under the influence of a road. Boxes represent variables; arrows represent causal effects; and labels on arrows represent processes involved in the effect. The total effect of the road is its direct effect plus its indirect effect on the environment.
The proposed causality behind road edge effects has implications for sampling design. On the one hand, comparisons among sites on a single side of the road are most prone to confusion between distance from the road, geographic position, and environmental gradients. On the other hand, comparisons between sites on opposite sides of the road allow both geographic position and the environment to vary for a given distance from the road, thus being more informative. Likewise, comparisons between sites along the road allow geographic position and environment to vary for the same distance from the road. However, in both cases, environment and geographic position can still correlate due to spatial autocorrelation, which is even more likely along very long roads since environmental heterogeneity increases with spatial extent (Leibold and Chase, 2018).
Researchers typically include environmental covariates in statistical models such as multiple regression to separate direct and indirect road effects (Ruffell and Didham, 2016; Ries et al., 2017). However, this does not control for confounding between environmental effects and spatial effects (i.e. dispersal limitation), nor guarantee that all environmental confounders have been measured; most likely, many confounders will not be measured simply because they are unknown (Shipley, 2016; Butsic et al., 2017; Arif and MacNeil, 2022). This way, two conclusions emerge: (1) regression-based estimates of road edge effects are easily biased; and (2) common sampling designs are unable to isolate road edge effects, although this might be possible with quasi-experimental designs (Butsic et al., 2017; Huntington-Klein, 2022; see below).
Road barrier effects on community dissimilarityRoads have also been widely studied as barriers to animal movement (Coffin, 2007; Fahrig and Rytwinski, 2009; Caplat et al., 2016). Roads could be dispersal barriers either because certain species avoid them (e.g. forest specialists) or because their individuals die while attempting to cross from one side to another (Laurance et al., 2009). However, roads are seldom absolute barriers; rather, they are permeable and some species, especially generalists, may benefit from roads and other linear clearings by their individuals using them as defecation sites, foraging trails, or dispersal corridors (i.e. road attraction) (Suárez-Esteban et al., 2013).
Dispersal limitation implies an increase in compositional dissimilarity between sites (Tuomisto and Ruokolainen, 2006). If species have the same probability of being limited by a road, compositional dissimilarity between sites on opposite sides of the road should increase relative to that between sites on the same side, as different species should be barred on each side by chance. However, species often vary in their response to roads. For instance, if roads select for species which are more likely to survive dispersal across them, this could decrease rather than increase compositional dissimilarity between opposite roadsides, as the same species would be favored on each side. Likewise, avoidance of roads by certain species should decrease their relative abundance on both roadsides, further decreasing compositional dissimilarity between them. This could be tested by comparing compositional dissimilarity between opposite roadsides among species groups that differ in their response to the road (e.g. avoidance vs. attraction, or high vs. low mortality by roadkill).
Inference on the barrier effect can be confounded by the cooccurrence of edge effects. For instance, if the edge effect is symmetric between roadsides, sites near the road should become more environmentally homogeneous, thus decreasing the environmental distance between sites on opposite roadsides. Consequently, compositional dissimilarity between roadsides could decrease in response to this environmental homogenization, which is contrary to what is predicted by the barrier effect. Thus, edge and barrier effects are naturally confounded in the context of roads. Likewise, geographic distance simultaneously affects the probability of being on opposite sides of the road, the environmental distance between sites (including environmental gradients that already existed before the road), and compositional dissimilarity itself (through isolation by distance). Thus, as with the edge effect, the potential for confounding is high when comparing compositional dissimilarity on opposite roadsides vs. on the same roadside (Fig. 2).

Causal diagram showing expected relationships between compositional dissimilarity, roadside, environmental distance, and geography distance across community pairs under the influence of a road. Boxes represent variables; arrows represent causal effects; and labels on arrows represent processes involved in the effect. The total effect of the road is its direct effect plus its indirect effect through environmental distance.
Roads may span large spatial extents, encompassing substantial environmental heterogeneity and variation in use intensity. In this context, we suggest that the most informative metacommunity is not the entire set of local communities along the road’s path; rather, it is the set of local communities around some section of the road, either adjacent to or physically intersected by the road. Accordingly, the ecologically relevant question would be: how the occurrence or some feature of the road would affect the metacommunity dissimilarity, i.e. the total or average dissimilarity among local communities within the metacommunity? For simplicity, we will consider metacommunities with similar area and shape, so that the degree of isolation by distance within them is constant.
Several factors are known to influence metacommunity dissimilarity, e.g. environmental heterogeneity, size and functional diversity of the species pool, and mean community size (Hubbell, 2001; Vellend, 2016; Leibold and Chase, 2018). Roads may add to or modify these effects through at least two ways: by physically crossing the metacommunity habitat, or through the intensity of road use in the segment where the metacommunity is located. As discussed earlier, road crossings could have barrier and edge effects within the metacommunity, which could either increase or decrease metacommunity dissimilarity. At the same time, road-use intensity could amplify both the barrier effect and the edge effect. Thus, any observed change in metacommunity dissimilarity will be the net result of these effects occurring across the local communities composing the metacommunity.
Yet, roads may also indirectly affect another important property of metacommunities: mean community size, or the average number of individuals in a local community. For instance, roadkill could drive source–sink dynamics that reduce population size of certain species (Fahrig and Rytwinski, 2009). Likewise, changes in the mean environmental conditions or in the environmental heterogeneity of the metacommunity could either reduce or increase mean community size, depending on how they affect species. Mean community size controls the strength of ecological drift: metacommunities with smaller mean community size should experience faster local extinctions by chance, thus increasing metacommunity dissimilarity (Hubbell, 2001; Hanson et al., 2012; Vellend, 2016). Ecological drift is also predicted to modify the effects of selection and dispersal. First, smaller mean community size should weaken environmental selection (Vellend, 2016; Jacobi and Siqueira, 2023), i.e. weaken the relationships between metacommunity dissimilarity and environmental heterogeneity across metacommunities (or the relationship between pairwise dissimilarity and environmental distance within metacommunities). Second, ecological drift should strengthen the effect of dispersal limitation, by accelerating the divergence between isolated communities through local random extinctions (Hubbell, 2001; Hanson et al., 2012; Vellend, 2016). Thus, in metacommunities under a road barrier effect (e.g. metacommunities crossed by a road, or in highly used road sections), metacommunity dissimilarity could increase due to dispersal limitation, but this effect should be stronger where mean community size is smaller.
More generally, road-use intensity, mean environmental conditions and their heterogeneity, and mean community size may all be influenced by geographic position along the road. For instance, road-use intensity may depend on proximity to human settlements, attributes of the road (e.g. paved vs. dirt, lighting, number of lanes, among others) or preferred transport routes. Mean environmental conditions and their heterogeneity may be spatially autocorrelated, e.g. due to the geological history of the region. In turn, both road-use intensity and the environment can affect mean community size. Likewise, dispersal limitation along great highways, for example, could generate gradients in mean community size, regardless of road use intensity and the environment. Thus, again, there is high potential for confounding when inferring road effects on metacommunity dissimilarity from correlations (Fig. 3).

Causal diagram showing expected relationships between mean compositional dissimilarity, mean community size, road use intensity, and environmental and geographic factors across metacommunities on different sections of a road. Boxes represent variables; arrows represent causal effects; and labels on arrows represent processes involved in the effect. The total effect of the road is its direct effect plus its indirect effects through mean community size and the environment.
The current standard for causal inference in science is the randomized controlled experiment (Shipley, 2016; Huntington-Klein, 2022; Siegel and Dee, 2025). To determine a treatment effect, treatment is randomly assigned among sampling units, creating statistical independence between the treatment and any other variable that could also affect the response, thus eliminating confounding. However, with observational data, this is generally impossible since the “treatment” (e.g. proximity to a road) could not be randomly assigned; rather, it typically correlates with many other variables that could also affect the response of interest, which can be unmeasured or even unknown. Furthermore, even if we could measure them, controlling for certain variables may introduce bias depending on how they are causally related (e.g. collider bias) (Shipley, 2016; Arif and MacNeil, 2022; Huntington-Klein, 2022; Siegel and Dee, 2025). Although the distinction between direct vs. indirect road effects on communities has been recognized in the ecological literature (Ruffell and Didham, 2016; Ries et al., 2017), the more general issue of causal identification has received limited attention (Butsic et al., 2017; Arif and MacNeil, 2022; Siegel and Dee, 2025).
Observational data can allow causal inference with quasi-experimental designs (Butsic et al., 2017; Huntington-Klein, 2022; Siegel and Dee, 2025). These designs use some source of exogenous variation to isolate the effect of interest: variation that affects the predictor of interest (e.g. distance from road) but does not affect any other variable that could also influence the response variable of interest (e.g. species composition). In a randomized experiment, the exogenous variable is the randomization itself: a binary, random variable which determines who receives the treatment (1) or not (0). In observational studies, exogenous variation can be found in some natural but specific contexts (Butsic et al., 2017; Huntington-Klein, 2022; Siegel and Dee, 2025). Historically, these designs have been more popular in sciences studying human populations (e.g. economics, epidemiology), where the required data may be easier to obtain.
One popular quasi-experimental design is Difference-in-Differences (DiD) (Butsic et al., 2017; Huntington-Klein, 2022; Siegel and Dee, 2025). In its simplest form, DiD is similar to the “Before-After Control-Impact” design (BACI) sometimes used by ecologists (Underwood, 1992). In DiD, one would sample community composition in sites near (treatment) and far from a road (control), before and after road construction/pavement (treatment event). Then, one would check if the treatment and control groups had similar temporal trends in composition before road construction (the “parallel trends assumption”). If this assumption is supported, and if no other confounder temporally coincides with road construction, any difference in temporal trends after road construction can only be caused by the road, even if treatment correlates with spatial confounders. This is typically tested with a regression model that includes an interaction between treatment (e.g. near road vs. far from road) and time (e.g. before vs. after road construction). Average differences between sites are controlled using the sampling sites as a categorical predictor (fixed effects), while heteroskedasticity and within-site temporal autocorrelation are accounted for using clustered standard errors (Huntington-Klein, 2022). The latter only adjusts the uncertainty about coefficients (not their point estimates) and thus is more conservative than assuming some explicit form for heteroskedasticity and autocorrelation, such as in the Generalized Linear Mixed Models (GLMM) often used by ecologists (Byrnes and Dee, 2025). Certainly, sampling more times before road construction can provide a stronger test of the parallel trends assumption.
As a practical example, a recent study used DiD to test for an effect of road construction on landscape descriptors in Wuhan, China (Tan and Zhou, 2023). They compared 5 km² blocks with vs. without new roads from 2005 to 2019. Interestingly, DiD revealed no road effect on the landscape metrics, whereas a standard regression did indicate an effect, suggesting bias due to unmeasured confounders. More generally, DiD is flexible and its analysis is an active area of research. For instance, the treatment can be continuous rather than binary, e.g. geographic distance from a road (although causal identification in such cases can be more difficult; Zhang, 2025). Further, sampling more times after road creation allows estimation of how the effect changes over time (e.g. delays), also called dynamic DiD or Event Study. If the parallel trends assumption does not hold, it can still be statistically mimicked with more flexible models, e.g. counterfactual estimators, which create control observations from model predictions based on untreated observations only (Liu et al., 2024). A practical limitation is that sampling biodiversity in tropical forests typically depends on access by roads (Carvalho et al., 2023), which may limit reaching relevant control sites, as big areas with continuous forest. Controls may be usually set inside protected areas, or non-protected areas accessed through large rivers. Therefore, access to remote areas, far from major rivers and roads, requires air manned aircrafts or remotely operated vehicles, which in themselves demand enormous financial resources, as well as complex logistics in terms of training, security, and field maintenance (Qi et al., 2026). This type of logistics is still an obstacle for most research projects.
Alternatively, many existing roads have been abandoned and are expected to be pavemented in the near future (Laurance et al., 2009). Instead of using new roads as treatment, one could use new pavement as treatment and before pavement as a control. Data on species composition for different sites at different times is increasingly available from public databases, and species composition of some taxa may be monitored with remote sensing (Wallis et al., 2017). More generally, these ideas also apply to questions at the metacommunity level. The barrier effect could be tested by comparing metacommunity dissimilarity between metacommunities traversed vs. not traversed by a road, before and after road construction or pavement.
DiD is just one of a family of quasi-experimental designs (e.g. regression discontinuity, instrumental variables) (Butsic et al., 2017; Huntington-Klein, 2022; Siegel and Dee, 2025). However, all such designs have specific assumptions that may or may not apply to a particular ecological question. Whether each of them applies to road ecology deserves further study.
Challenges and opportunities to infer road effects in tropical forests: the case of BR-319 in Brazilian AmazoniaManaus city, capital of the Brazilian state of Amazonas, is an important economic center in the Amazonia region and currently the largest city in the whole region (2.2 million inhabitants). However, until the beginning of the 1970s, Manaus was considered isolated, as there were no terrestrial roads connecting this city to the rest of Brazil (Jesus et al., 2022). The only way to access the city was via aquatic or aerial transportation. Furthermore, Amazonas state politicians had issues with the Brazilian Military Dictatorship at the time, which had invested more in infrastructure and economic activities in the neighboring state of Pará than in Amazonas (Fearnside and de Alencastro Graça, 2006). Therefore, the Military Dictatorship decided to build a highway, the so-called BR-319, that would connect Manaus to the rest of the country and vice versa. This road would be 885 kilometers long and would start in Manaus and end in Porto Velho, the capital of the neighboring state of Rondônia, to the south (Jesus et al., 2022).
This road was inaugurated in 1976 by the Brazilian Military Dictatorship. However, due to severe climate conditions and the lack of maintenance by the federal government, this road became impassable from 1988 onwards. The southern section of the road (between the cities of Porto Velho and Humaitá) has remained passable for approximately 200 km. The north section of the road (between Manaus and Careiro Castanho, approximately 125 km) is also passable. However, a stretch in the middle of the route remains impassable, although occasional convoys of vehicles have made the journey at the height of the dry season in some years (bridges have been maintained to allow access to microwave towers along the route) (Fearnside and de Alencastro Graça, 2006; Ferrante et al., 2021; Fearnside, 2022). Currently, BR-319 is in the midst of a debate between those who argue that this road should be rebuilt and paved with asphalt and those who claim that this reconstruction could bring enormous impacts to the entire Western Amazonia (Ferrante et al., 2021; Fearnside, 2022).
The existence of road recovery plans raises concerns among environmentalists because the restoration tends to facilitate access to the region and result in extensive deforestation and forest degradation (Fearnside and de Alencastro Graça, 2006). With viable traffic on the highway, the deforestation projected for the next 20 years suggests a reduction in the original forest cover by at least 16.6%, in addition to threatening another approximately 44% of forested area located around the BR-319 that represent areas outside protected areas (Graça et al., 2014).
Most ecological studies carried out along the BR-319 highway so far have identified significant correlation between changes in species composition and environmental variables (Baccaro et al., 2013; Marciente et al., 2015; Schietti et al., 2016). These findings may overemphasize the role of natural selection, even though there is evidence that processes related to dispersal (Stegmann et al., 2019) may also be important in that region. However, these studies have often examined these processes individually, failing to consider their interaction or independence (see Abreu et al., 2018 for an exception). For example, the distribution of dung beetle species along the road is mainly correlated with the depth of the water table, the proportion of clay and silt in the soil (Salomão et al., 2022); however, it is known that these environmental variables are not uniformly distributed along the highway (Cintra et al., 2013; Ferreira et al., 2020), which could subject metacommunities on different sections of the road to different assembly rules. Testing whether species are absent from other locations due to dispersal limitation (Hargreaves et al., 2014; Lee-Yaw et al., 2016) or examining the possibility that ecological drift could also contribute to compositional dissimilarity between communities (Jacobi and Siqueira, 2023) could enhance our understanding of road effects on community assembly. That said, conclusions about community assembly along the BR-319 highway are so far based on correlative analyses with high potential for confounding, as discussed before. Hence, basic questions such as the strength and extent of edge effects and the degree to which the road limits dispersal remain unanswered.
Yet, the BR-319 highway is exceptional in that it already shelters a research infrastructure for ecological studies, implemented by the Brazilian Program for Biodiversity Research (PPBio) and the Long-term Ecological Project (PELD) (see da Rosa et al., 2021; Bergallo et al., 2023). There are 11 sampling modules distributed along both sides of the road. Each module follows the RAPELD sampling design, a framework for standardized, integrative sampling of ecological data (Bergallo et al., 2023). Each site has two parallel 5-km long trails, with a 250-m sampling transect located perpendicularly at each 1 km along each trail (thereby totalling 10 transects per module). Transects follow terrain contour lines to standardize altitude, thus minimizing soil and other environmental characteristics within transects relative to their variation among transects. Transect width is variable, being adjusted to the organism or variable of interest. Modules are adjacent to the road, so that all transects of a given site are on the same roadside but vary in their distance to the road from a few hundred meters to several kilometers (Fig. 4). Additionally, modules can be thought of as different metacommunities along the road, potentially experiencing very different assembly rules. For instance, the road encompasses large-scale gradients in soil, vegetation and climate through the Purus-Madeira interfluve (Schietti et al., 2016), and there are known gradients in animal abundance (e.g. bats; Marciente et al., 2015). The relative importance of selection to compositional dissimilarity may vary depending on local environmental heterogeneity, whereas the relative importance of ecological drift should vary with mean community size. Different sections of the road vary in intensity of use, with sections closer to its paved and more used borders in the northern and in the southern, whereas the central segment remains an unpaved dirt road, which could change the strength of any barrier effect (Da Rosa and Bager, 2013).

Although modules could be thought of as blocks that allow controlling for between-module confounders (Byrnes and Dee, 2025), this does not control for confounding between road distance, environmental gradients and geographic position within modules. The DiD design could be used to compare transects varying in distance from the road before and after asphalt pavement, or to compare within-module dissimilarity between modules with vs. without asphalt pavement, before and after the asphalt pavement. This is important because paved roads increase the roadkill risk given the higher traffic volumes and speed compared to non-paved ones (Santos and Ascensão, 2019). As no modules are traversed by the road and no modules directly face each other, the current design is more limited to test for a barrier effect; species composition can be compared between modules on opposite roadsides, but this is subject to unknown environmental confounders that correlate with roadside, as discussed before. Yet, new modules, paired with existing ones and on their opposite roadside, could be established in sections where pavement is planned and where it is not. This would allow directly estimating compositional dissimilarity between roadsides for sections with vs. without pavement, before and after the new pavement, providing a strong test of the barrier effect.
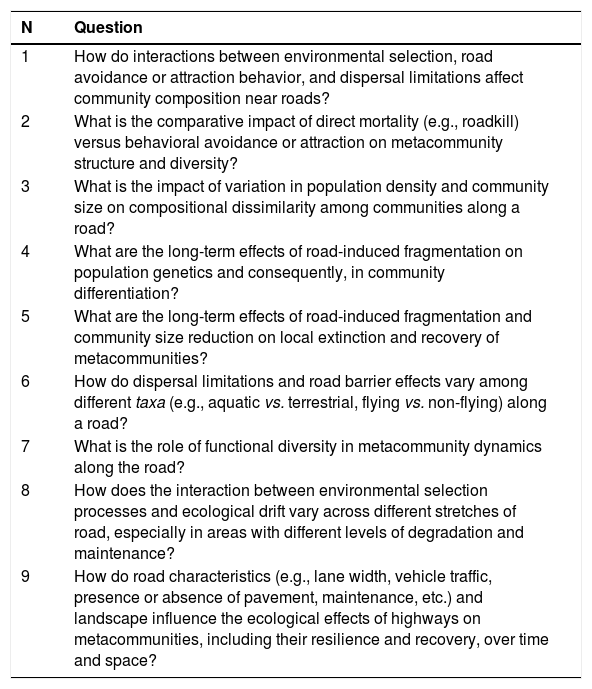
Final remarksGiven the environmental changes and anthropogenic pressures along all tropical roads, including the BR-319, tailored interventions based on a deeper understanding of how roads affect community assembly processes could be invaluable for biodiversity conservation. We suggested key questions addressing the most important gaps on roads and metacommunities in the tropics that we discussed along the text and that remain unanswered for the majority of the great roads built so far (Box 1). Additionally, these insights have the potential to inform and influence public policy, providing a scientific basis for decisions aiming to protect the Amazonian biodiversity. This reflects the broader necessity for a more integrated, multi-process approach to studying species communities, that goes beyond merely describing correlations to identify the causality of ecological processes, not only for the Amazonia but also for other ecologically sensitive regions. Future investigations along the BR-319 highway should strive for a comprehensive understanding that integrates various ecological processes and their interactions, considering both spatial and temporal dimensions. It's important to emphasize that Amazonia shelters different native people and has a key role when it comes to climate regulation and epidemiologic issues. This way, the progress presented by the South American governments as infrastructure implementation for socioeconomic development in wild preserved areas can cost more than money for us as humankind.
Key questions highlighted by BR-319 studies that could enhance our understanding how roads affect community assembly patterns
| N | Question |
|---|---|
| 1 | How do interactions between environmental selection, road avoidance or attraction behavior, and dispersal limitations affect community composition near roads? |
| 2 | What is the comparative impact of direct mortality (e.g., roadkill) versus behavioral avoidance or attraction on metacommunity structure and diversity? |
| 3 | What is the impact of variation in population density and community size on compositional dissimilarity among communities along a road? |
| 4 | What are the long-term effects of road-induced fragmentation on population genetics and consequently, in community differentiation? |
| 5 | What are the long-term effects of road-induced fragmentation and community size reduction on local extinction and recovery of metacommunities? |
| 6 | How do dispersal limitations and road barrier effects vary among different taxa (e.g., aquatic vs. terrestrial, flying vs. non-flying) along a road? |
| 7 | What is the role of functional diversity in metacommunity dynamics along the road? |
| 8 | How does the interaction between environmental selection processes and ecological drift vary across different stretches of road, especially in areas with different levels of degradation and maintenance? |
| 9 | How do road characteristics (e.g., lane width, vehicle traffic, presence or absence of pavement, maintenance, etc.) and landscape influence the ecological effects of highways on metacommunities, including their resilience and recovery, over time and space? |
The authors declare that they have no known competing financial interests or personal relationships that could have appeared to influence the work reported in this paper.
This work was supported by the Coordination of Superior Level Staff Improvement (CAPES) [scholarship number 88887.925766/2023-00]; the National Institute for Science and Technology INCT-SinBiAm [CNPq Nº 406767/2022-0 and 382946/2024-3]; INCT-CENBAM [CNPq number 406474/2022-2 and 01.02.016301.02394/2024-50]; CAPES/FAPEAM [scholarship number 88887.964874/2024-00]; the Program for Biodiversity Research (PPBio) of the Brazilian Ministry of Science, Technology and Innovation (MCTI) [CNPq Nº 441260/2023-3 e 441228/2023-2] and the Long-Term Ecological Research Program in the Southwest of Amazonas (PELD-PSAM) [Nº 021/2020; CNPq Nº 441366/2020-1 e 445988/2024-0]; the Fundação de Amparo à Pesquisa do Estado do Amazonas [scholarship FAPEAM/PROFIX-RH – Nº 009/2021, number 01.02.016301.00407/2022-94 and FAPEAM/PRODOC Nº 016/2023], the Franco-Brazilian Center for Amazonian Biodiversity (CFBBA), the French Embassy in Brazil, the French National Institute for Sustainable Development (IRD), Dr. Stéphanie Jacquet and the Infectious Diseases and Vectors Ecology Genetics Evolution and Control (MIVEGEC) Research Unit [mobility grant 2025].